


 Espanhol (pdf)
 Artigo em XML
 Referências do artigo

 Tradução automática
 Enviar este artigo por email
 Citado por SciELO
 Similares em
SciELO

 Permalink


Introduction
The reproductive study of animals used in the livestock industry is part of the success of these systems (Madhusoodan et al., 2019). Bull fertility is important in the development of the productive systems (Waberski et al. 2021, Barth, 2018), and their evaluation allows one to select those animals with better reproductive conditions (Petrunkina et al., 2007) or discard animals or ejaculates with poor quality parameters that could be infertile or subfertile. A bull’s seminal quality could be influenced by multiple factors, such as season (Barth, 2018), health (Taylor et al., 2018), nutrition (Cheah & Yang, 2011), animal species (Castellini et al., 2011), and semen conservation (Awad, 2011).
Bull semen preservation is usually associated with assisted reproduction techniques in which the spermatozoon is generally frozen. However, subjecting the cells to this process can affect their characteristics, this limiting their functionality when they are subsequently thawed (Awad, 2011). Sperm morphometry is a cell characteristic that can be used as an indicator for potential freezability or male fertility (Maroto-Morales et al., 2016; Villaverde-Morcillo et al., 2017).
Sperm morphometry is usually determined by performing the CASA-Morph module (Gallagher et al., 2018; Mortimer & De Jonge, 2018; Valverde et al., 2019a; 2019b), which allows one to analyze characteristics related to the size and shape of the head, acrosome, and intermediate piece of the sperm (Vicente-Fiel et al., 2013; Yániz et al., 2015). These characteristics may differ according to the method of cell fixation (Soler et al., 2015), staining (Banaszewska et al., 2015; Boersma et al., 1999), and evaluation systems (Vicente-Fiel et al., 2013). Morphometry is relevant because it could be used to predict the fertility potential of males (Franken, 2015; Toner et al., 1995) and to explain alterations of cells caused by the spermiogenesis process (Valverde et al., 2016), as well as explain some relationships with other sperm variables (Giaretta et al., 2017; Hook & Fisher, 2020). Despite the importance of this analysis, its use has been characterized by variability in evaluation and methodologies (Garcia-Herreros et al., 2006).
For this reason, these variations in the morphometry of sperm cells have been analyzed and distinct characteristics have been determined in the ejaculate of the same animal (Buchelly Imbachí et al., 2022; Martínez-Pastor, 2022). Therefore, using cluster analysis allowed us to identify different subpopulations with an ejaculate based on the data from the CASA systems (Barquero et al., 2021; Martínez-Pastor, 2022; Valverde et al., 2016; Yániz et al., 2018). These new analyses have favored the explanation of the conformation of the ejaculates and their relationship with the potential fertility of the animals analyzed (Santolaria et al., 2015).
On the other hand, sperm morphometric characterization could be used to distinguish animal species (Sampaio et al., 2017). Sperm morphometry differences have been observed when comparing different species of foxes (Andraszek et al., 2020), ovine (Martínez-Fresneda et al., 2019), neotropical primate (Sampaio et al., 2017), and even dog breeds (Soler et al., 2017a). In the literature, there are separate studies of sperm morphometry for both B. taurus and B. indicus, but there are only a few that compare them within the same study (Beletti et al., 2005) .To our knowledge, no study has compared sperm morphometry between B. taurus taurus and B. taurus indicus using a CASA-morph system and subpopulation analyses.
Therefore, the aim of this study was to determine different sperm subpopulations based on morphometry parameters of frozen-thawed semen in two bovine subspecies using a CASA-morph system.
Methodology
The study was conducted using cryopreserved straws and doses were supplied by Avance Genético S.A. (Alajuela, Costa Rica). The study was conducted from May to December 2023, at the Animal Reproduction Laboratory (AndroTEC), located at the Campus Tecnológico Local San Carlos (CTLSC), in Santa Clara, Florencia, Alajuela, Costa Rica (CRTM05; X: 444296 Y: 1146016). Ethical approval was granted by the Committee of Centro de Investigación y Desarrollo de la Agricultura Sostenible para el Trópico Húmedo at the Costa Rica Institute of Technology (CIDASTH-ITCR) under Section 20/2023, Article 1.0, reference DAGSC-188-2023 and CIE-206-2023 Section 20-2023, Article 3.19.
Animals, semen collection and processing: Semen was collected from 5 Simmental (Bos taurus) bulls and 5 Brahman (Bos indicus) bulls with an average age of 5.7±2.8 and 3.6±1.6 years respectively, by artificial vagina under a collection program of two times per week. The semen samples were assessed for volume by conical tube graduated at 0.1 mL and concentration using a bovine photometer Accucell (IMV, L’Aigle, France) at 530 nm wavelength. Semen was diluted using a commercial extender OptiXcell® (IMV, L’Aigle, France), with a ratio depending on ejaculate volume. In any case, the final concentration given with the diluent was 25×106 cells/straw. The equilibrate procedure consist in a decrease slowly at a rate of −0.3°min−1 until 4 °C of the diluted semen, after these were maintained at the same temperature for 4-5 hours. The semen was packed in 0.25 mL straws with an automatic filling and sealing machine (MRS1, IMV Technologies, L’Aigle, France). Then, the straws were frozen in a programmable freezer, (Digitcool 5300, IMV, L’Aigle, France) at the following rates: 4 to −10°C at 5°C min−1,
−10 to −100°C at 40°C min−1, and −110 to −140°C at 20°C min−1. Finally, the straws were stored by plunging into liquid nitrogen.
Sperm sample preparation for morphometric analysis: Sperm morphometric analysis was performed slides from straws for each bull. In a slide a previously mixed subsample of 10 μL extended were placed, extended and identified. The samples were stained with the Diff-Quik® kit (Medion Diagnostics, Düdingen, Switzerland) following all the manufacturer’s instructions step by step. The slides were then kept for the subsequent double-blind scheme analysis.
Morphometric assessment systems: Morphometric evaluations of semen were performed using the ISAS®v1 (Integrated Semen Analysis System, Proiser R+D, Valencia, Spain) using the parameters that the software brings by default. The images capture was made using a digital video camera (Proiser 782 m, Proiser R + D) connected to a UB203 microscope (UOP/Proiser R + D) with a 100× bright field objective and an attached 3.3× pho to-ocular. The camera video frame grabber array size was 746 × 578 × 8 bit, using 256 gray levels with 0.084 μm/pixel resolution available in both axes of the analysis images. A minimum of 200 images of different spermatozoa were captured and analyzed. The spermatozoon was capture randomly, discriminated these if there were particles that potentially interfered with the sperm head boundary. In case of an erroneous definition of the sperm head boundary, the system allowed us to vary the analysis factor and if not was possible to analyze a correct boundary, the cell was deleted from the analysis. A graphical schematic of the experimental design is shown in Figure 1.
Morphometric variables: Eight sperm head morphometric variables were analyzed, divided into four parameters of head size (length (L, μm), width (W, μm), area (A, μm2 ), and perimeter (P, μm)) and four head shape parameters derived from the head size (ellipticity (L/W), rugosity (4πA/P2 , elongation ((L−W)/(L+W)), and regularity πLW/4A)) were also obtained. All the data obtained from each sperm were saved in an Excel® (Microsoft Corporation, Redmond, Washington, USA) for further analysis.
Statistical analysis: Data for all sperm variables were assessed for homoscedasticity using Levene tests and for normality using a normal probability plot. An identity link function with a normal distribution was assumed for all sperm morphometric response variables. ANOVA was applied to evaluate statistical differences between treatments for these variables. Post-hoc pairwise comparisons between species means were conducted using the Tukey- Kramer test.
Multivariate procedures: Multivariate procedures were employed to identify sperm clusters from the subset of sperm morphometric data. To mitigate scaling effects, all morphometric variables were standardized. Principal factor analysis (PFA) was conducted to derive a few linear combinations that retained most variance of the original variables’ information. Prior communalities were estimated using the maximum absolute correlation coefficient between each variable and others. The number of principal factors (PFs) extracted was determined using the Kaiser criterion, selecting those with eigenvalues >1. The dataset’s adequacy for factor extraction was assessed using the KMO (Kaiser-Meyer-Olkin) statistic (Spencer, 2013). Varimax rotation with Kaiser normalization (Kaiser, 1958) was applied.
A two-step cluster procedure was performed using the sperm-derived indices obtained from the principal component analysis (PCA). Sperm morphometric measurements within each ejaculate were clustered based on shape and size parameters using a non-hierarchical K-means clustering procedure with the Euclidean distance metric (Kaufman & Rousseeuw, 1991). The analysis identified sperm subpopulations and detected outliers. ANOVA was applied to evaluate statistical differences between clusters for all morphometric variables, with significance defined at P < 0.05. Pairwise comparisons between cluster means were conducted using the Tukey-Kramer test. Results are presented as mean ± standard error of the mean. All data were analyzed using IBM SPSS, version 23.0, for Windows (SPSS Inc., Chicago, IL, USA).

Figure 1 Bovine sperm morphometric assessment procedure. (1) Ejaculates were obtained from two bull groups (n = 5 per group) and packaged as sperm doses. (2) Doses were cryopreserved using an automated freezing protocol. (3) For analysis, frozen doses were thawed (30 s at 37 °C), smeared on slides, and stained with the morphometric stain described in the Methods. (4) At least 200 sperm heads per sample were digitally imaged and analyzed using a computer‑assisted morphometry system to generate four size and four shape descriptors of the sperm head (see Materials and Methods for parameter definitions).
Analysis and results
Some previous research has demonstrated the adverse effects of cryopreservation on semen quality (Maroto-Morales et al., 2016). The cryopreservation process has an important impact on sperm morphology (Awad, 2011) and potential fertilization capacity (Franken, 2015), so it has a very specific effect on the proportion of spermatozoa that make up the different subpopulations (Rubio-Guillén et al., 2007). The decrease in the percentage of sperm with long and large sperm heads, and the increase in the proportion of cells in the smaller sperm subpopulation is a known consequence of cryopreservation (Gravance et al., 2009). This effect may directly condition the results observed in this work, based on the evidence that European breeds may have greater tolerance to cryopreservation processes (Saranholi et al., 2021). However, this factor would also imply that the decrease in the morphometric parameters of one subspecies compared to another causes an effect on the distribution of subpopulations, since, when evaluating other variables such as kinetics, some changes are observed as reported in previous studies (Víquez et al., 2020).
It has been reported that sperm morphometry can be affected by different factors, such as osmotic pressure, staining techniques, freezing and thawing (Caldeira et al., 2022; García-Molina et al., 2023; Soler et al., 2017a; Soler et al., 2017b; Soler et al., 2005, 2016; Soler et al., 2017c; Valverde et al., 2019; Yániz et al., 2016). These variables can have a significant impact not only on sperm dimensions (Awad, 2011), which could lead to inaccurate assessment, but also on chromatic structure, which can have direct negative implications on the individual’s fertility potential (Banaszewska et al., 2015). Results of this work allow us to understand more about the variations that could occur in the morphometric characteristics of spermatozoa between the different bovine subspecies.
Differences between species indicated that genotype composition influenced the value of each sperm head size and shape variable. When the sperm head length was studied, samples from B. taurus (9.007 ± 0.037 μm) were the longest (p < 0.05) compared to those obtained from B. indicus (8.969 ± 0.026 μm). Width values differed (p < 0.05) according to species, in decreasing order, of B. taurus (4.886 ± 0.016 μm), and B. indicus (4.756 ± 0.011 μm). The head area of spermatozoa in both B. taurus or B. indicus was not different (p > 0.05). There were differences in head sperm perimeters (p < 0.05) when comparing the use of taurus and B. indicus species. In relation to head shape variables, the values oscillated differently in both species (Table 1).
Table 1 Morphometric variables (mean ± SEM) of bull sperm size and head shape of in two different bovine subspecies.
| Variables | Bos indicus | Bos taurus |
|---|---|---|
| Length | 8.969 ± 0.026b | 9.007 ± 0.037a |
| Width | 4.756 ± 0.011b | 4.886 ± 0.016a |
| Area | 37.120 ± 0.124 | 37.792 ± 0.172 |
| Perimeter | 24.767 ± 0.048b | 24.791 ± 0.068a |
| Ellipticity | 1.896 ± 0.006a | 1.846 ± 0.009b |
| Rugosity | 0.761 ± 0.001b | 0.772 ± 0.002a |
| Elongation | 0.307 ± 0.002a | 0.296 ± 0.002b |
| Regularity | 0.901 ± 0.002b | 0.915 ± 0.003a |
Note: SEM: standard error of the mean. Length (L, μm), width (W, μm), area (A, μm2), perimeter (P, μm), ellipticity (L/W), rugosity (4πA/P2), elongation ((L − W)/(L + W)), regularity (πLW/4A). a-b Different letters indicate differences between ejaculate sub-populations for morphometric variables. p < 0.05.
Source: own study.
Heterogeneity in mammalian ejaculates could explain the behavior of species and their evolution according to the conditions in which they have developed ( & Van Look, 2004; Ramón et al., 2014 as this has allowed us to understand how different types of spermatozoa different functions within the ejaculate could have to achieve successful reproduction of the species (Ramón et al., 2014). Morphomet ric evaluations between the subspecies taurus and Bos indicus showed differences in sperm size and shape characteristics. This coincides with previous research that has determined that sperm from zebu bulls tend to be smaller in size compared to other breeds, including European breeds (Beletti et al., 2005).
Three PC factors were identified. In B. indicus, PC1 was found to be positively associated with ellipticity and elongation, and negatively related with the rugosity parameter. PC2 was related to perimeter and area. PC3 was related to shape variable regularity. In the B. taurus, PC1 was found to be related to head size (area, width, and perimeter, in decreasing order) and PC2 was associated with shape head (ellipticity, elongation and regularity and, to a lesser degree, length). PC3 was negatively related with regularity. The total variance explained was 95.39 %, and 90.798 % for B. indicus and B. taurus, respectively (Table 2).
Table 2 Eigenvectors of principal components (PCs)* for the morphometric variables of bull sperm size and head shape in bovine subspecies.
| Variable | ||||||
|---|---|---|---|---|---|---|
| Bos indicus | Bos taurus | |||||
| PC1 | PC2 | PC3 | PC1 | PC2 | PC3 | |
| Length | 0.703 | 0.765 | ||||
| Width | 0.898 | |||||
| Area | 0.929 | 0.949 | ||||
| Perimeter | 0.915 | 0.892 | ||||
| Ellipticity | 0.983 | 0.810 | ||||
| Elongation | 0.984 | 0.808 | ||||
| Rugosity | -0.886 | |||||
| Regularity | 0.995 | 0.804 | -0.828 | |||
| Var Exp | 52.772 | 27.114 | 15.503 | 36.317 | 32.628 | 21.853 |
Note: Var Exp: variance explained in each PC. Total variance explained: Bos indicus = 95.389 %; Bos taurus = 90.798 %. *Indicates the more important variables in each PC. Only eigenvectors > 0.6 are presented.
Source: own study.
This discovery underscores the importance of further investigating the genetic mechanisms responsible for these differences for a thorough understanding of how breed genetics can shape sperm characteristics as a measure of adaptation. These results suggest that the cryopreserved materials of Bos indicus and Bos taurus could have three sperm subpopulations according to their shape and size. Other researchers have studied the relationship that the shape and size of sperm could have with evolutionary mechanisms of different species (Kramer et al., 2024). In addition, other studies found in the literature comparing the morphometric characteristics of Bos taurus and Bos indicus and suggest that the differences could be associated with individual characteristics of the animals and their fertility (Beletti et al., 2005) and that they could be related as a function of membrane and acrosome quality (Palacin et al., 2020).
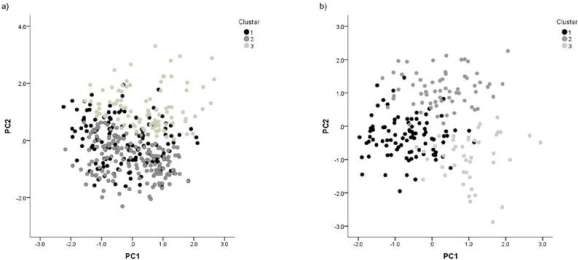
Principal components identify three subpopulations in B. indicus: SP1 with 32.9 % of the total spermatozoa, SP2 with 43.0 % of the cell analyzed in this species, and SP3 with 24.1 % of the total spermatozoa. For B. taurus, three subpopulations were found: SP1 contained 46.0 % of the sperm cells. SP2 had a total of 32.0 % of the male gamete. The last subpopulation (SP3) was comprised of 22.0 % cells (Figure 2).
Note. Source: own study.
Figure 2 Interactions between principal components (PCs) for the morphometric variables of bull sperm size and head shape by bovine subspecies. a) Bos indicus, b) Bos taurus.
The distribution was not the same for each species but there were differences in subpopulations within each species (p < 0.05), and the distribution was not the same for each species. Results from B. indicus indicated differences between subpopulations upon comparison. SP1 was characterized by the medium size (length and area), while SP2 was characterized by the smallest cells and SP3 showed the highest spermatozoa size. Similarly, results described in B. taurus indicate that sperm subpopulations were different (p < 0.05). SP1 was characterized by the smallest cells, and the head shape wasthe intermediate for all variables, except for the rugosity value, which was the highest. SP2 and SP3 were high, with the highest values of each variable oscillating from one to the other. In both species, a different composition was observed, with SP3 having the highest head size values, except for the length. The shape variables in B. taurus indicate that SP1 and SP2 values were different to SP2 and SP3 for B. indicus (Table 3).
Table 3 Morphometry of sperm heads and head shape variables (mean ± SEM) of bull semen sub-populations (SPs) in different bovine subspecies.
| Variables | Bos indicus | Bos taurus | ||||
|---|---|---|---|---|---|---|
| SP1 | SP2 | SP3 | SP1 | SP2 | SP3 | |
| Length | 9.110±0.031ar | 8.634±0.027bt | 9.273±0.036cx | 8.581±0.040as | 9.768±0.048bu | 9.009±0.057cy |
| Width | 4.888±0.016ar | 4.678±0.013ct | 4.821±0.018bx | 4.726±0.023as | 4.829±0.028bu | 5.068±0.034cy |
| Area | 37.272±0.126ar | 35.941±0.109bt | 39.381±0.147bx | 35.232±0.240as | 39.068±0.288bu | 40.485±0.347cy |
| Perimeter | 24.733±0.050ar | 24.246±0.043bt | 25.678±0.058cx | 23.851±0.082as | 25.532±0.098bu | 25.815±0.118bx |
| Ellipticity | 1.875±0.010br | 1.856±0.009at | 1.934±0.012cx | 1.818±0.009as | 2.025±0.011bu | 1.780±0.013cy |
| Rugosity | 0.766±0.002br | 0.768±0.002ct | 0.752±0.002ax | 0.778±0.003as | 0.753±0.003bu | 0.764±0.004cy |
| Elongation | 0.301±0.002br | 0.297±0.002at | 0.315±0.003cx | 0.290±0.002as | 0.338±0.003bu | 0.280±0.003cy |
| Regularity | 0.937±0.002ar | 0.881±0.002bt | 0.889±0.002cx | 0.904±0.003as | 0.949±0.004bu | 0.886±0.005cx |
Note: SEM.: standard error of the mean. Length (L, μm2), width (W, μm), area (A, μm2), perimeter (P, μm), ellipticity (L/W), rugosity (4πA/P2), elongation ((L − W)/(L + W)), regularity (πLW/4A). a-c Different letters within species indicate differences between ejaculate sub-populations for morphometric variables. r-s Different letters within SP1; t-u within SP2; and x-y within SP3 indicate differences between bull species for morphometric
variables. p < 0.05.
Source: own study.
Cluster analysis has shown that bull ejaculates are not homogeneous in terms of sperm population (Martínez-Pastor, 2022), and the distribution of spermatozoa also varied between subspecies. Results showed the presence of subpopulations with wide variability in both B. taurus and B. indicus bulls. These findings suggest that the differences could be related to genetics between these two subspecies, evidence that points towards the possibility that race-associated genetics could exert a significant influence on the observed variations in sperm morphometry (Terán et al., 2021; Thurston et al., 2002). Despite this, it is necessary to further investigate the possible implications of these genetic differences and their relevance on other sperm variables as an adaptation mechanism of each subspecies to conditions that affect the reproductive success of livestock.
Conclusions
The variability in semen morphometry analysis underscores the need to standardize semen evaluation protocols. This approach has revealed differences in sperm characteristics between subspecies, such as B. taurus and B. indicus, indicating potential genetic influences. Furthermore, the cryopreservation process itself introduces changes in sperm morphology, which begs for a comprehensive understanding of its effects on different sperm subpopulations.
Funding
This research was funded by Costa Rica Institute of Technology (Vice-Chancellor’s office of Research and Extension; VIE (Vicerrectoría de investigación y Extensión); Project VIE-2151083. The APC was funded by Costa Rica Institute of Technology (Vice-Chancellor’s office of Research and Extension; VIE (Vicerrectoría de investigación y Extensión) and by AGROALNEXT programme (Agroalnext/2022/063; European Union NextGenerationEU (PRTR-C17.I1), Generalitat Valenciana).
Acknowledgements
The authors thank the Costa Rica Institute of Technology (ITCR) for financing this study. This work was supported Costa Rica Institute of Technology (Vice-Chancellor’s office of Research and Extension; VIE (Vicerrectoría de investigación y Extensión; Project 2151083 “Optimización de la conservación y búsqueda de parámetros de la fertilidad en espermatozoides de animales de interés productivo”)) and Postgraduate Office of ITCR. The funders had no role in the study’s design, data collection, and analysis, decision to publish, or preparation of the manuscript.
Author contribution statement
Conceptualization, A.V., M.A.S; methodology, F.S., L.V., A.V.; software, F.S., L.V., J.S., I.A.Z.; validation, F.S, A.V.; formal analysis, A.V.; investigation, F.S., L.V., I.A.Z.; resources, A.V.; data curation, F.S., L.V., , I.A.Z; writing-original draft preparation, F.S., A.V., I.A.Z.; writing-review and editing, F.S., A.V., J.S., M.B., M.A.S., C.D.C.; visualization, A.V.; supervision, A.V.; project administration, A.V.; funding acquisition, A.V., M.A.S.. All authors have read and agreed to the published version of the manuscript.

