


 Inglés (pdf)
 Articulo en XML
 Referencias del artículo

 Traducción automática
 Enviar articulo por email
 Citado por SciELO
 Similares en
SciELO
 uBio

 Permalink

Introduction
In Central America, large tracts of forest are suffering a drastic reduction due to the advance of the agricultural frontier and the expansion of human settlements (Kaimowitz, 1996), as well as the effects of activities related to mining and wood extraction ( et al., 2001). Costa Rica has an area of 1 152,150 ha for the sustainable production of wood, corresponding to the humid tropical forest and rainforest from the Huetar Norte, Atlántico and La Brunca regions (Chassot, 2006). Here, a selective harvest scheme has been implemented, and legislation establishes a minimum of 15 years between harvests (Publicación No. 27388-MINAE, N° 212, 1998). This time allows a wood volume to recover to ensure long-term production, but little is known about whether this period is sufficient for the recovery of animal communities (Sánchez Núñez, 2009).
The compatibility between forest harvesting and biodiversity conservation has been questioned because forest logging can have direct or indirect adverse effects on the components and attributes of biodiversity (Putz et al., 2001). Forest harvesting directly alters the structure and composition of the forest and can cause fragmentation, resulting in a landscape with fewer and more isolated forest fragments (Mason & Thiollay, 2001). Forest products and by-products have disrupted the remaining forests, which could change bird communities and populations and their infectious agents (King et al., 2010). When resources, including food, are reduced in an area, birds may gather in larger flocks more often (Zhou et al., 2010), even close to farms, favoring the transmission of diseases between species. This can lead to disease outbreaks if suitable conditions for individual species (Daszak et al., 2000).
This study aimed to compare the presence of ecto and endoparasites, Chlamydia psittaci, Borrelia spp., Anaplasma spp., and Rickettsia spp. in birds and their ticks inhabiting forest fragments with different degrees of alteration (with or without forest harvesting, and embedded in landscapes with different agriculture amount) in northern Costa Rica, to provide valuable data for understanding host-parasite relationships and the influence of habitat conditions on them. The results are interpreted in terms of national regulations about forest harvesting, providing information that can help improve harvesting schemes and habitat protection and developing preventive measures.
Materials and methods
Study area: The study was conducted in the Northern Huetar Conservation Area of Costa Rica from February 2008 to June 2010. We selected nine forest units according to their degree of alteration, defined by the type of forest management in each forest unit (two classes, harvested or non-harvested) and the amount of agriculture in 500ha area surrounding each forest unit (2 classes, high or low crop intensity). Harvested forests were operated by the Commission on Sustainable Forestry Development of San Carlos (CODEFORSA) in the early 90’s and have not been harvested between then and the date of this study. Therefore, these forests have undergone approximately 20 years of natural recovery at the time of this study. Non-harvested forests are some of the few remaining preserved forests in the area and have never been harvested.
We created a hexagonal grid and overlaid it on land use and cover to calculate the agricultural area in each 500ha cell. So, each hexagon covered 500 hectares and included both the forest fragment and its surrounding matrix. This spatial configuration ensured uniform sampling units and reduced edge effects commonly associated with square grids. The study area was then classified according to the agricultural amount in each hexagon cell to visually examine the distribution of agricultural lands (ESRI, 2009). We used this information to select forest units for sampling in zones with either high or low crop intensity as an additional criterion to the type of forest management. Consequently, we selected both harvested and non-harvested forest units in areas with high crop intensity or low crop intensity. We run variance models in R to corroborate the difference in the amount of agriculture surrounding forest units (R Core Team, 2013). Mean agriculture field was more extensive in an area of 500ha surrounding forest units allocated to "high crop intensity" class (171,39ha; 95%: 83,04 - 259,74ha) than "low crop intensity" class (49.09ha; 95%: 32,65 - 80,86ha) classes (F=11,46, P= 0,0117). As a result, we considered four harvested forests and five non-harvested forests. Besides, five of these forests belonged to the low crop intensity class and four to the high crop intensity (Fig. 1).
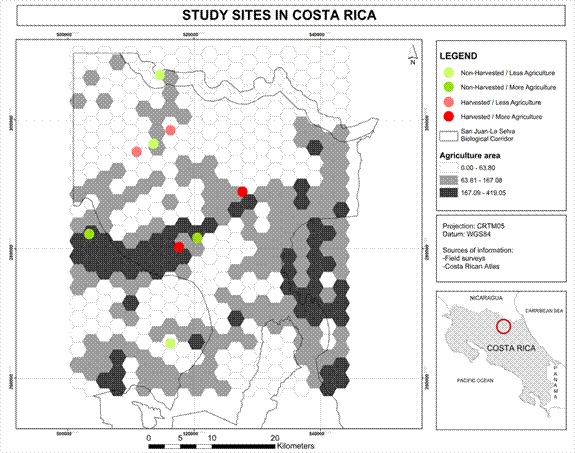
Fig 1 Study sites classified according to forest harvesting and fragmentation in the Northern Huetar Conservation Area of Costa Rica.
Bird sampling: We placed eight mist nets (12 x 2,5m and 32mm) along transects spaced 100m apart in each one of the nine sampling sites from February 2008 to June 2010. They were checked for netted birds at 30-min intervals from 5:30 am until 10:30 am. Each mist-netting session lasted one week. Captured birds were identified by species, banded, and visually examined for body condition, ectoparasites, and lesions. Ectoparasites from feathers were picked off and stored in ethanol 70%. Feces, blood samples, and oropharyngeal and cloacal swabs were collected from some birds (Table 1). Samples were stored at 4 °C in the forest and promptly transported to the Veterinary School of the Universidad Nacional de Costa Rica, where they were kept at -20°C. Recaptured individuals were released immediately.
Table 1 Samples collected and analyzed to determine infectious agents
| Target of Analysis | Sample Type | Number of Samples or Individuals |
| Ectoparasites | Mites, lice, and ticks (nymphs, larvae, and adults) | 555 ectoparasites (409 mites, 25 lice, and 121 ticks) from 407 birds |
| Endoparasites | Feces | 147 |
| Chlamydia spp. | Cloacal and oropharyngeal swabs | 221 and 225, respectively |
| Rickettsia spp., Anaplasma spp., and Borrelia spp. | Ticks | 121 |
Parasitological analysis: We collected feathers from a subsample of 407 birds on which ectoparasites were visible when they were handled. Feathers were examined for mites, lice, and ticks (nymphs, larvae, and adults). Mites, lice, and ticks were mounted on Hoyer medium. The feces were analyzed using the flotation technique with a hyper-saturated sugar solution. The taxonomic identification of ectoparasites was carried out at the genus level (Atyeo & Braasch, 1966; Clay, 1953; Mironov, 1985; Nava et al., 2017; Orwig, 1968; Park & Atyeo, 1971). Likewise, the endoparasites were also classified at the genus level, except for one group classified at the order level (Larki et al., 2018; Tenter et al., 2002; Yamaouti, 1961). The number of positives for each parasite type was recorded.
Molecular analysis: We analyzed oral and cloacal swabs for Chlamydia spp., while ticks were analyzed for Rickettsia spp., Anaplasma spp., and Borrelia spp. According to the manufacturer's instructions, DNA extraction from swabs and ticks were performed using the DNeasy Blood & Tissue Kit (QIAGEN, Chatsworth, CA, USA). A set of already published primers was selected to identify bacterial species (Table 2). The following positive controls were used: DNA of C. psittaci, donated by the Clinic of Birds, Reptiles, Amphibians and Fish, Justus Liebig University, Giessen, Germany; DNA of A. phagocytophilum (strain Trestom) HL-60 infected cells, donated by the CDC Atlanta, USA; DNA of Borrelia burgdorferi s.l. donated by the Center for Biomedical Research of La Rioja, Spain, and DNA from R. felis. All PCR experiments included water (Fermentas®) used as a negative control. Reactions were performed with Dream Taq PCR Master Mix 2X (Fermentas), primers (0,1𝜇M), DNA (∼20𝜇g), and water (molecular biology grade, Fermentas). PCR products were visualized by agarose gel electrophoresis (1,4%) in TBE (Tris Base, boric acid, EDTA, pH8, 0,5 M), and ethidium bromide staining (0,5g/ml). GeneRuler 100 bp DNA Ladder Plus (Sm0321, Fermentas®) was used for DNA sizing.
Table 2 Protocols used for determining infectious agents
| Pathogen | Protocol | Primer Name | Sequences (5'-3') |
| Chlamydia spp. | (Kaltenboeck et al., 1991) | 191CHOMP CHOMP371 | GCIYTITGGGARTGYGGITGYGCI AC TTAGAAIC(GT)GAATTGIGC(AG)(TC)IA GTGIGCIGCTT |
| Rickettsia spp. | (Labruna et al., 2004) | CS-78 CS-323 | GCAAGTATCGGTGAGGATGTAAT GCTTCCTTAAAATTCAATAAATCAGGAT |
| (Regnery et al., 1991) | Rr190.70p Rr190.602n | ATGGCGAATATTTCTCCAAAA AGTGCAGCATTCGCTCCCCCT | |
| Anaplasma spp. | (Alberti et al., 2005) | EphplgroEL (569) EphplgroEL (1193) | ATGGTATGCAGTTTGATCGC TCTACTCTGTCTTTGCGTTC |
| A. phagocytophilum | (Massung et al., 1998) | Ge3a Ge10r Ge9f Ge2 | CACATGCAAGTCGAACGGATTATTC TTCCGTTAAGAAGGATCTAATCTCC AACGGATTATTCTTTATAGCTTGCT GGCAGTATTAAAAGCAGCTCCAGG |
| Borrelia burgdorferi sensu lato | (Rijpkema et al., 1995) | 23SN1 23SC1 23SN2 5SCB | ACCATAGACTCTTATTACTTTGAC TAAGCTGACTAATACTAATTACCC ACCATAGACTCTTATTACTTTGACCA GAGAGTAGGTTATTGCCAGGG |
Note: derived from research.
Genomic DNA was extracted from tick pools with Blood and Tissue kit (Qiagen, Hilden, Germany) according to the manufacturer's instructions. PCRs protocols for rickettsial agents were detailed in a previous report (Dolz et al., 2019).
Statistical analysis: We conducted statistical analyses in R (R Core Team 2013). We used analysis of variance (ANOVA) models to compare the number of bird species, total number of individuals, and the Shannon diversity index across two categorical factors: harvest condition (harvested vs. non-harvested) and agricultural intensity (high vs. low). For more complex relationships, we fitted generalized linear mixed models (GLMMs). These models included harvest condition and habitat fragmentation class as fixed effects, while the site was included as a random effect to account for repeated measures or spatial clustering. Response variables in GLMMs included bird richness, abundance, and Shannon index, using appropriate distributions (e.g., Poisson or Gaussian) according to the nature of each variable. Additionally, to assess the relationship between ectoparasite load and land-use factors, we constructed separate generalized linear mixed models (GLMMs) with ectoparasite presence or counts as the response variable, and harvest condition and agricultural intensity as fixed effects, with site again treated as a random effect. We also examined model residuals to ensure that the assumptions of normality and homoscedasticity were met, and we selected the final models based on AIC values.
Results
We captured 838 birds from 76 spp. 460 birds from 58 species belonged to non-harvested sites, and 378 birds from 50 species to harvested sites. Although non-harvested sites presented a higher number of bird species and a higher number of individuals than harvested sites, these differences were not statistically significant (F=2,322, P= 0,171, and F=0,064, P= 0,808, respectively). In addition, 460 birds from 59 species belonged to sites with less agriculture, and 378 birds from 47 species to sites with high crop intensity. Although units with low crop intensity presented a higher number of bird species and more individuals than units with high crop intensity, these differences were also not statistically significant (F=0,002, P= 0,969, and F= 0,064, P= 0,808, respectively). On the other hand, the Shannon diversity index was higher in harvested than in non-harvested sites and in units with low crop intensity than in units with high crop intensity. However, these differences were not statistically significant (F= 2,893, P= 0,133, and F= 0,027, P= 0,875, respectively) either.
A total of 555 ectoparasites (409 mites, 25 lice, and 121 ticks) were collected from 407 birds. Percentages of infection (PI) of 4,2% (17/407), 59,5% (242/407), 18,0% (73/407), and 9,1% (37/407) were established for the mites of the Analges, Pterodectes, Proctophyllodes, and Trouessartia genera, respectively; while PI of 6,1% (25/407) for Rallicola lice, and 12,5% (51/407) for Amblyomma ticks were determined. Only Amblyomma spp. larvae and nymphs were collected on 47 birds. A higher proportion of Proctophyllodes sp. was found in non-harvested sites (Z= -0,0081081, p-value <0,05). According to the amount of agriculture, Analges spp. (Z = -0,027027, p-value <0,05) and Pterodectes spp. (Z=-0,250614, p-value <0,05) presented a higher proportion in units with low crop intensity. However, Trouessartia spp. (Z=0,056511, p-value <0,05) and Amblyomma spp. (Z= 0,066339, p-value <0,05) showed a higher proportion in units with high crop intensity (Table 3).
Table 3 Avian ectoparasites in nine forest sites from the Northern Huetar Area in Costa Rica
| Forest | Percentage of birds infected | |||||
| Mites | Lice | Ticks | ||||
| Analges spp. | Pterodectes spp. | Proctophyllodes spp. | Trouessartia spp. | Rallicola spp. | Amblyomma spp. | |
| Harvested | 2,2 (9/407) | 30,7 (125/407) | 4,9 (20/407) | 8,4 (34/407) | 3,2 (13/407) | 5,7 (23/407) |
| Non harvested | 2 (8/407) | 28,7 (117/407) | 13 (53/407) | 3,2 (13/407) | 2,9 (12/407) | 6,9 (28/407) |
| Total | 4,2 (17/407) | 59,5 (242/407) | 18 (73/407) | 9,1 (37/407) | 6,1 (25/407) | 12,5 (51/407) |
| High crop intensity | 0,7 (3/407) | 17,2 (70/407) | 8,6 (35/407) | 8,6 (35/407) | 3,2 (13/407) | 9,6 (39/407) |
| Low crop intensity | 3,4 (14/407) | 42,3 (172/407) | 9,3 (38/407) | 2,9 (12/407) | 2,9 (12/407) | 2,9 (12/407) |
| Total | 4,2 (17/407) | 59,5 (242/407) | 18 (73/407) | 9,1 (37/407) | 6,1 (25/407) | 12,5 (51/407) |
Of the total of the fecal samples 11,6% (17/147) were positive for endoparasites. Coccidia (Eimeria spp. and Isospora spp.) were the most frequent protozoan found in fecal samples (9,5%), while nematodes such as Strongylida and Echinuria spp. were only slightly represented. The frequencies of endoparasites were not significantly different between harvest or fragmentation groups (Table 4).
Table 4 Percentage of avian endoparasites found in feces in nine forest sites from the Northern Huetar Area in Costa Rica.
| Forest | Coccidia | Strongylida | Equinuria spp. |
| Harvested | 3,4 (5/147*) | 0,7 (1/147) | 0,7 (1/147) |
| Non harvested | 6,1 (9/147) | 0,7 (1/147) | 0 (0/147) |
| Total | 9,5 (14/147) | 1,4 (2/147) | 0,7 (1/147) |
| High crop intensity | 5,4 (8/147) | 0 (0/147) | 0,7 (1/147) |
| Low crop intensity | 4 (6/147) | 1,4 (2/147) | 0 (0/147) |
| Total | 9,5 (14/147) | 1,4 (2/147) | 0,7 (1/147) |
*Total of birds from which feces were obtained
A total of six Amblyomma spp. ticks were positive for Rickettsia spp. These positive cases were found in the non-harvested/low crop intensity, non-harvested/high crop intensity, and harvested/high crop intensity categories. All the birds belonged to the order Passeriformes and fed on insects from the understory of humid forests, including old-growth secondary forests (Table 5). On the other hand, ticks were negative for Anaplasma spp. and Borrelia spp. Neither the 221 oropharyngeal samples nor the 225 cloacal samples collected from birds were positive for C. psittaci.
Table 5 Description of bird species with Rickettsia spp. positive ticks.
| Forest sites | Type of site | Bird species | Bird family | Migration status | Conservation status | Food habits |
| Golfito | Harvested / High crop intensity | Attila spadiceus Catharus ustulatus | Tyrannidae Turdidae | Resident Migratory | Low concern | Insects, spiders, small frogs, lizards, berries and seeds Fruits, seeds, some insects and invertebrates |
| Santa Helena | Non- harvested / High crop intensity | Dendrocincla fuliginosa | Furnariidae | Resident | Low concern | Insects and spiders |
| Chacha -lacas | Non- harvested / Low crop intensity | Glyphorhynchus spirurus Thamnophilus atrinucha Phaenostictus mcleannani | Furnariidae Thamnophili dae Thamnophili dae | Residents | ND Low concern Low concern | Insects and spiders Insects, spiders, and lizards Insects, spiders, scorpions, other invertebrates and small vertebrates |
Note: Mixed generalized linear model results are included as supplementary data.
Discussion
Habitat loss and fragmentation are among the primary causes of biodiversity loss, increasing the risk of species extinction (Fahrig, 2003). Forest harvesting has been related to changes in the components and attributes of biodiversity (Putz et al., 2001), which are conditioned by factors such as the ecological requirements of the species (Woltmann, 2000), the intensity of harvesting (Mason, 1996), and logging schemes and techniques (Bawa & Seidler, 1998).
In Costa Rica, a selective harvesting scheme has been implemented, and legislation establishes a minimum of 15 years between harvests. One study in northern Costa Rica forest fragments found that the estimated richness of birds and number of individuals per trophic guild showed no significant differences between harvested (16 years previous to the study) and non-harvested forests (Sánchez Núñez, 2009). However, these parameters tended to be higher in non- harvested forests. Nevertheless, species composition varied between forests: non-harvested forests had more species of hummingbirds, nuthatches, antbirds, and psittacine than harvested forests. Species occurrence for all trophic guilds differed between non-harvested and harvested forests, with this parameter tending to be greater in non-harvested forests. Sánchez Núñez (2009) stated that these harvested forests seemed to be recovering after harvesting, although more research was needed to ensure sufficient time for a total recovery of bird communities after forest harvesting. Similarities found in this study in the number of bird species, total number of individuals, and Shannon diversity indices between harvest or fragmentation classes seem to agree with those found by Sánchez Núñez (2009).
Concerning parasite infection of birds in northern Costa Rica, mites were the most common ectoparasites found in this study, similar to previous reports (Enout et al., 2012). However, we found a low percentage of chewing lice. In Costa Rica, Rallicola ochrolaemi, R. fuliginosa, and R. cephalosa were reported previously in bird species such as Automolus ochrolaemus, Dendrocincla fuliginosa, and Glyphorynchus spirurus (Sychra et al., 2007). On the other hand, we found a higher tick infestation rate of birds (12,5%) than the 7% reported by other authors in different wild birds in seven protected areas on the Caribbean and Pacific slopes of Costa Rica (Ogrzewalska et al., 2015). A low percentage of coccidian parasites was found, while other studies have reported Eimeria and Isospora as common and occasional (Cole & Friend, 1999). Time of day, age, and feeding habits affect coccidian oocyst shedding in wild passerines, with more of these parasites found in the afternoon (López et al., 2007). However, these captures were carried out in the morning. It is also possible that physiological differences in feeding habits between species could have affected these results (Boughton, 1933; Dolnik, 1999a, 1999b). Additionally, gastrointestinal parasites are not excreted constantly, and the use of a single fecal sample per bird may have limited the detection of these parasites; serial sampling would have been ideal but was not feasible under the conditions of this field study.
Six ticks (Amblyomma spp.), found in six different birds, were positive for Rickettsia amblyommatis. These ticks were found in three forest sites: two in forests surrounded by high crop intensity areas and one in a forest surrounded by low crop intensity areas. Other researchers have proposed that a higher prevalence of ectoparasites (in this case, ticks) on birds in fragmented areas of Brazil might be caused by the dominance of a few generalist bird species in small patches, allowing easier transmission of parasites among individuals (Ogrzewalska et al., 2011). In addition, in more fragmented areas, we might expect a more heterogeneous landscape, with forest fragments interspersed with other classes of land use, for example, pastures for cattle or other productive uses. This might, in turn, maximize contact not only among individuals of wildlife species in forest fragments but even between wildlife and domestic animals living in the matrix surrounding forest fragments. This scenario may increase access to cattle and cattle ticks (Tolesano-Pascoli et al., 2010), which is relevant considering all avian species with Rickettsia spp. positive ticks usually visit the ground to seek food or collect material to build nests (Sick, 1997).
A non-expected pattern was found in the case of ectoparasite infection and Rickettsia spp. positives in areas with or without forest harvesting; two of the three forest sites with ticks positive for Rickettsia spp. were found in non-harvested sites and one in a harvested site (harvested at least 15 years before sampling). It might be expected that birds inhabiting forests subjected to disturbances by logging would be more stressed or have lower immune defenses (Klukowski & Nelson, 2001; Tieleman et al., 2005), which might, in turn, affect their parasite load and lead to increased prevalence of a disease agent in the environment (Deem et al., 2001; Patz et al., 2000).
In addition, according to the dilution effect, we might expect a higher proportion of parasites in more disturbed and possibly less diverse forests, such as harvested areas (Ostfeld & Keesing, 2000). However, a higher proportion of Proctophyllodes sp. in non-harvested forests was found. Moreover, a higher diversity of birds was found in the harvested forest than in the non- harvested forest, although this difference was not statistically significant. However, the intermediate disturbance hypothesis may be considered here - a mechanism proposed by Connell (1978), to explain the maintenance of diversity in tropical forests and coral reefs. This hypothesis states that intermediate disturbance in mature ecosystems maintains higher levels of species richness and biodiversity than in the absence of such disturbances (Roxburgh et al., 2004). The similarity of bird richness and diversity among forest sites, and the absence of disease agents in birds found in this study, may account for a tendency towards recovery taking place in bird communities of harvested forests from northern Costa Rica, given the selective forest harvesting scheme and the period between harvests (16 years) applied to these forests. However, it is necessary to identify consequences in the birds' health when forests are harvested and in the first years following that harvesting.
The other infectious agents (Anaplasma spp. and Borrelia spp.) analyzed in ticks were negative in this study. In Europe, Borrelia burgdorferi s.l. was found and transmitted, especially by Ixodes ricinus ticks (Gern et al., 1998), which are reported in the highlands of Costa Rica (Ogrzewalska et al., 2015). We also obtained negative results for chlamydiosis in birds. Studies around the world on chlamydiosis in Passeriformes are not common, mainly because they are not considered to play an important role in the transmission of the bacteria (Kaleta & Taday, 2003). However, a few studies have reported these species as carriers of the bacterium (Olsen et al., 1998; Rehn et al., 2013; Simpson & Bevan, 1989).
In general, the bird communities analyzed in this study might be diverse enough to dilute the probability of the presence of most of the infectious agents analyzed, consistent with the dilution effect (Ostfeld & Keesing, 2000). These authors suggested that habitat loss and fragmentation can contribute to disease outbreaks indirectly through the loss of biodiversity while maintaining high biodiversity might decrease the prevalence of an infectious disease among hosts due to the dilution effect. It is also possible that the avian communities in this study were similar because they were in a similar and relatively small landscape, probably shaped by the same biophysical factors and human productive activities. Future studies that consider a larger number of forest sites in areas showing much larger differences in forest size and fragmentation may provide further insights into the effects of habitat loss and fragmentation on disease ecology.
These results seem to support the dilution effect proposed for the effects of habitat fragmentation on disease transmission. However, the forest sites analyzed were similar in terms of health status and the presence of disease agents in birds. This may reflect a possible tendency towards recovery in the harvested forests studied or a strong similarity among forest sites because of their closeness in a generally similar landscape.
Ethics, conflict of interest, and funding statement
The authors declare that we have fully complied with all pertinent ethical and legal requirements, both during the study and in the production of the manuscript; that there are no conflicts of interest of any kind; that all financial sources are fully and clearly stated in the acknowledgements section; and that they fully agree with the final edited version of the article. A signed document has been filed in the journal archives.
The statement of each author’s contribution to the manuscript is as follows: All co-authors: Study design. K.B.P., A.E.J.R., and G.D.: Laboratory analysis. M.R.I.: Data collection and analysis. All co-authors: preparation and final approval of the manuscript.

