




 Inglês (pdf)
 Artigo em XML
 Referências do artigo

 Tradução automática
 Enviar este artigo por email
 Citado por SciELO
 Similares em
SciELO
 uBio

 Permalink


Introduction
Ecological-interactions studies among closely related species, particularly within a particular habitat, have a long history in ecology (MacArthur, 1958; Miller, 1967; Pianka, 1994). This has been a central issue to understand habitat partitioning and competition among species, species-specific adaptive responses, and the importance of such interactions in shaping the evolution within a particular group of species (MacArthur, 1972; Ricklefs & Miles, 1994; Winkler & Leisler, 1985). For decades, interaction among closely related species spun around competition and niche partitioning. A large number of investigations have focused on measuring differences among species and attributing such differences to competition, without certainly tested if competition was the source of the differences detected, and much less, the effect of competition on species reproduction (Strong, 1984). Competition cannot be completely discarded as a potential factor influencing the coexistence of related species in a community, since in some groups of species competition has been important in shaping the structure of communities (Tilman, 1987; Tilman, 1994). However, in other cases careful conducted experiments demonstrated that competition was inexistent, in groups of species for which competition had previously been considered an important ecological factor shaping the communities (Wiens, 1989; Wise, 1993).
A more recent approach integrates morphology and ecology (competition included as a potential but not an exclusive factor) under an evolutionary framework to understand the habitat partitioning and foraging strategies of a group of closely related species (Losos, 1990a; Losos, 1990b; Losos 1990c; Losos & Miles, 1994; Norberg, 1994). This approach opened the opportunity to consider habitat (and niche) partitioning as an adaptive response of (individuals within species) species to variation in the environment, considering environment as the interaction between abiotic (e.g., vegetation structure, ambient temperature) and biotic factors (e.g., resource availability, predation). Within birds, new world warbles (Parulidae) are a group model that has been the focus of attention in competition and niche partitioning (MacArthur, 1958), and on their interaction with their tropical counterparts during the wintering season (Keast, 1980).
The mangrove warbler (Setophaga petechia erithachorides) is the only warbler present during the non-wintering season of North America migratory birds in Costa Rican mangroves (Barrantes, 1998). However, during the overwintering period, the mangrove warbler shared its habitat with large numbers of other warblers, including the yellow warbler (S. petechia). Yellow warblers consist of a large group of subspecies, including the mangrove warbler (Lowther et al., 1999). This particular condition permits the comparison of foraging strategies in a group of related birds inside of a relatively simple tropical forest, the mangrove forest. Additionally, the arriving of migratory warblers permits contrasting the foraging strategies of the mangrove warbler, and thus its flexibility (plasticity), between two very different conditions: being the only warbler in its habitat, and sharing the habitat with a large number of other family members. We specifically focus on answering the following questions: (1) Do the foraging strategies differ among five warbler species (Setophaga p. erithachorides, S. petechia, Protonotaria citrea, Parkesia noveboracensis, and Leiothlypis peregrina) in the mangrove forest? We particularly focus on two aspects of foraging strategies: the substrates use by warblers while foraging, and the maneuvers they use to attempting capturing prey. In this case we predict that those species more similar in morphology shared similar foraging strategies. (2) Do the mangrove warblers modify its foraging strategy when migratory warblers are present? We expect that if migratory warblers with similar foraging strategies are abundant, the mangrove warbler will modify its foraging strategy. A plastic response that allows mangrove warblers to reduce competition with other family members.
Material and methods
Description of the study area: We conducted this research from July 1986 to December 1987 in a mangrove forest in Chomes, Puntarenas, Costa Rica (10°, 02’ N; 84°, 54’ W). We delimited an area of 70 ha in which all data were collected. Climatically, the region is characterized by a long dry season, from December to May or June, with the rainy season that includes the other months (Epifanio et al., 1983).
The vegetation in the area vary according to the tides influence. The zone of greater influence includes trees of Rhizophora mangle, R. harrisonii, Avicennia germinans, A. bicolor, and Laguncularia racemosa (Jiménez & Soto, 1985), but in areas above the tides influence (or nearly so) plants such as Volkameria pittieri, Conocarpus erectus, Prosopis juliflora, Pithecellobium dulce, Capparis odoratissima and Cynophalla flexuosa are common.
Substrates and foraging maneuvers: To record the use that different warbler species made of the mangrove forest we defined six foraging substrates (Supplementary Table 1). The categorization of substrates was based on preliminary observations of warblers in the study area. To evaluate if each warbler species used a different set of maneuvers to capture prey, we defined 15 different maneuvers (Supplementary Table 1) based on preliminary observations of warblers in the study area and published information by Holmes et al. (1979); Fitzpatrick (1980); and Robinson & Holmes (1982). These maneuvers were defined as a combination of specific maneuvers on a particular substrate (Supplementary Table 1), following Fitzpatrick (1980), Holmes et al. (1979), and Remsen & Robinson (1990).
Table 1 Use of foraging substrates and foraging maneuvers by five warbler species (Setophaga p. erithachorides, S. petechia, Protonotaria citrea, Parkesia noveboracensis, and Leiothlypis peregrina) in a mangrove forest.
| A | Substrates use: all species | ||||
|---|---|---|---|---|---|
| Factor | DF | Sum of squares | R2 | F | P |
| Species | 4 | 12.31 | 0.76 | 80.41 | 0.001 |
| Residual | 102 | 3.90 | 0.24 | ||
| Total | 106 | 16.22 | 1.00 | ||
| B | Substrate use: excluding P. noveborascensis | ||||
| Species | 3 | 1.08 | 0.27 | 10.27 | 0.001 |
| Residual | 83 | 2.92 | 0.73 | ||
| Total | 86 | 4.00 | 1.00 | ||
| C | Foraging maneuvers: all species | ||||
| Species | 4 | 10.65 | 0.72 | 66.70 | 0.001 |
| Residual | 103 | 4.11 | 0.28 | ||
| Total | 107 | 14.76 | 1.00 | ||
| D | Foraging maneuvers: excluding P. noveborascensis | ||||
| Species | 3 | 0.88 | 0.25 | 9.15 | 0.001 |
| Residual | 83 | 2.66 | 0.75 | ||
| Total | 86 | 3.54 | 1.00 | ||
Collected and preparation of data: To compare the foraging pattern of each warbler species we collected data along transects haphazardly selected in the interior and border of the mangrove. All observations were collected from 630 to 1 200 h for 9 days every two weeks for a total of 39 sampling sessions. Prior to collect the information we created a unique letter code for substrates (e.g., a = trunk, e = foliage) and a unique numeric code for the maneuvers (e.g., 1 = gleaning, 2 = probing).
We used a voice recorder (Sony M-570V Handheld Cassette Voice) to collect the foraging activity of warblers. When a warbler was found foraging, we described to the voice recorder the sequence of different substrates and different maneuvers that the warbler used during the observation time. For instance, a sequence of a1-e2-a2 means that during the observation time the bird glean on a trunk, then probe in the foliage, and finally probe in a trunk. We then played back the tape to extract the time that each individual bird spent on each substrate and used each specific maneuver. For each individual we summed the effective time for each substrate and maneuver. We also had a code to indicate that the bird was inactive. This allowed us to subtract this time from the total time recorded for a specific individual and obtain the effective time.
For each individual of each species for which we obtained a foraging sequence, we calculated the weighted mean to compensate for differences in the total time we observed each individual. For example, if T 1 was the total effective time of the sequence of bird 1, S i the time the bird foraged in the substrate i, and ΣT the sum of the effective time of all birds of the same species in a particular sampling session, we calculated the weighted mean as: S i *T 1 / ΣT. We next sum the weighted means of all individuals of each species for each particular sampling session to have an entrance (row) for species for sampling session. This approach has two advantages; first, it compensates for differences in the effective time across individuals, making the data comparable across species; and second, we reduced the effect of pseudoreplicates, because it was likely that we recorded some of the same individuals in consecutive days in a sampling session. We used the same approach for the time warbles spent in each of the capturing maneuvers.
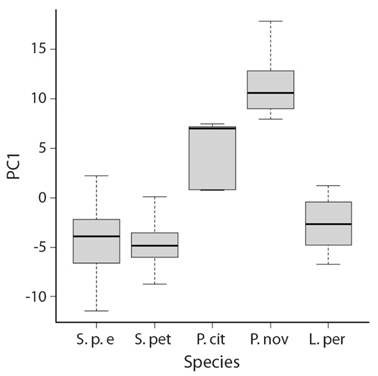
Morphological data: We obtained measurements of seven morphological traits 1) tarsus length (from the intertarsal joint to the middle of the sole of the foot), 2) wing chord length (unflattened), 3) tail length, 4) culmen length, 5) culmen width, 6) culmen depth, and 7) weight, from specimens of the same warbler species, from the ornithology collection of Museo de Zoología, CIBET, Universidad de Costa Rica. We performed a Principal Component Analysis on morphological traits to reduce the number of variables. The first component explained 81% of the variance corresponding to the seven morphological traits. Therefore, we used the first PCA as a proxy of the birds’ morphology for comparisons.
Statistical analyses: We used two different approaches to compare the use of substrates and capturing maneuvers across species. First, we compared the variation in time birds spent foraging in each substrate and using each capturing maneuver across species with the coefficient of variation (cv). Lower cv values indicate that birds used substrates or maneuvers more homogeneously.
Second, analyses of habitat use and foraging behavior include, in most cases, multiple variables, making univariate statistical analyses unpractical. Considering the type of data obtained in this study, we took a different approach. We used statistics designed for comparing species composition across communities, but instead of species abundances we fed the models with frequencies, specifically with the time (number of seconds) an individual of a given warbler species forage on each specific substrate or spend in each of the foraging maneuvers.
We constructed two matrices, one for substrates and another for maneuvers. The columns of these matrices consisted of either the substrates or the maneuvers, and the rows included several entries of each species. Each row including the number of seconds birds of a given species forage on each specific substrate or spend on each specific maneuver during each sampling session (see above).
To test for differences in substrates and maneuvers across species and for Setophaga p. erithachorides between seasons (presence vs. absence of migrants), we used the permutational analysis of variance (PEMANOVA) (vegan::adonis2; Oksanen et al., 2020). We tested for homogeneity of multivariate variances, using the vegan::betadisper function to test for equal dispersion in the data, and found homogeneous variances (P values ranged from 0.16 to 0.68) in all cases.
The morphology was compared among warbler species with a linear model. We included the PCA scores corresponding to the first component as the response variable and the species as the predictor. We then compared between species the PC1 means with the functions emmeans and pairs of the package emmeans (Lenth et al., 2018). We used the R statistical language for all analyses (R Core Team, 2024).
Results
General results: We collected information on foraging substrates and maneuvers employed to capture prey for 12 warbler species in the mangrove forest. However, only 5 species had enough sample size to be included in the analyses (Setophaga p. erithachorides, S. petechia, Protonotaria citrea, Parkesia noveboracensis, and Leiothlypis peregrina). The abundance of migrants fluctuated over the study period but it increased rapidly after the first arrivals, overpassing by far the number of S. p. erithachorides (Fig. 1).
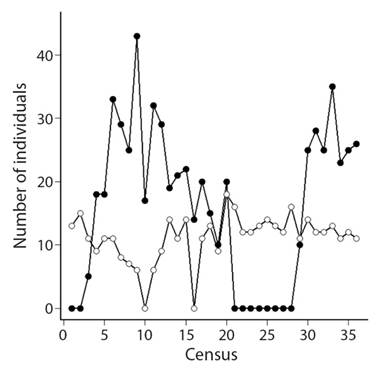
Fig. 1 Abundance of the four (S. petechia, P. citrea, P. noveroracensis, and L. peregrina) migrant warblers (black dots) and the resident S. p. erithachorides (white dots). The absence of migrants (0 individuals) is consequence of migrants flying to their breeding grounds in North America.
Foraging substrates and foraging maneuvers- all species: The time warblers foraged on each substrate varied widely across species (Supplementary Table 2), but with species aggregated in two groups. The first group included S. p. erithachorides, S. petechia and P. citrea which used the substrates more homogeneously (lower cv values) than the second group that included P. noveboracensis and L. peregrina (Fig. 2A).
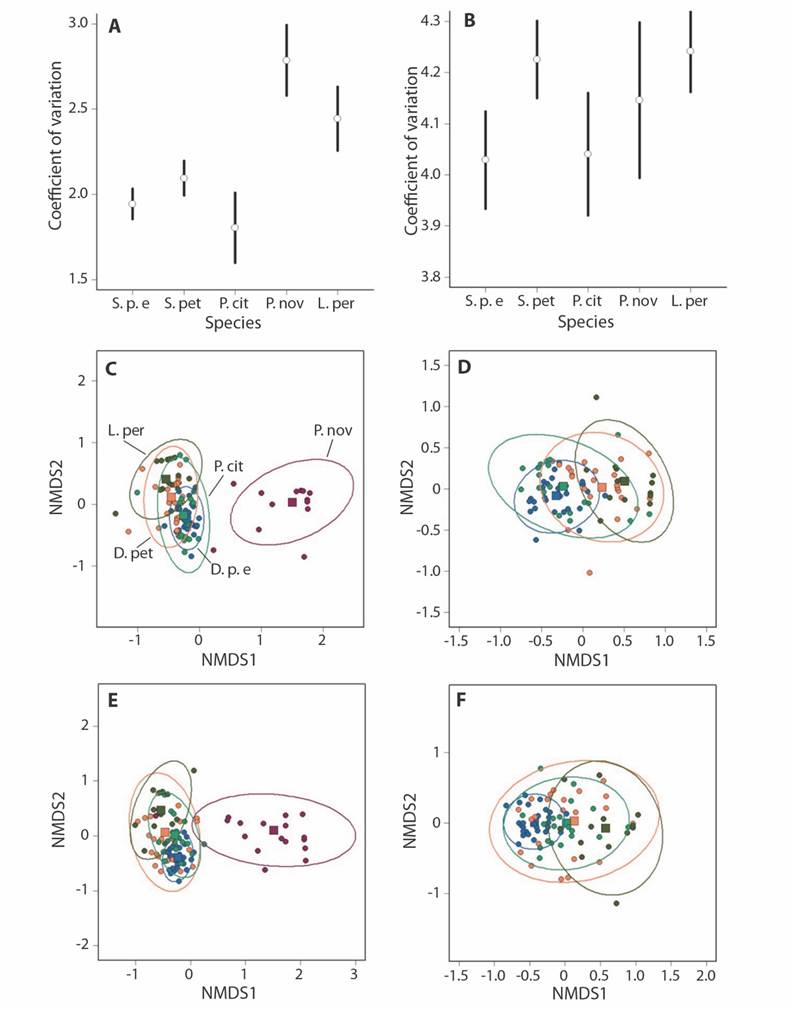
Fig. 2 Comparison of foraging strategies of the five warbler species: Setophaga petechia erithachorides (S.p.e), S. petechia (S.p), Protonotaria citrea (P.cit), Parkesia noveboracensis (P.nov), and Leiothlypis peregrina (L.pe). Coefficient of variation (mean and confidence intervals) calculated for the time warblers used the different foraging substrates (a) and the foraging maneuvers (b). Use of substrates by the five warbler species (c) and excluding P. noveboracensis (d). Use of foraging maneuvers by the five warbler species (e), and excluding P. noveboracensis (f). The squares represent the centroids and the ellipses are the 95% confident intervals.
The use of capture maneuvers was more heterogeneous than the use of substrates as indicated by higher values of the cv (Fig. 2B; Supplementary Table 3), but there were some patterns. Two of the species (S. petechia and L. peregrina) had higher mean cv values, indicating an even more heterogenous used of maneuvers than S. p. erithachorides and P. citrea; with P. noveboracensis having a larger variation in maneuvers used across foraging sessions. Hence, P. noveboracensis and L. peregrina showed a narrower preference for substrates than the other warblers, and S. petechia and L. peregrina showed a narrower preference for maneuvers (Fig. 2A-B).
The use of substrates (analyzed with PERMANOVA) also indicated a marked difference across species (Table 1A; Fig. 2C). Parkesia noveboracensis differed notably from the other warblers that showed a larger similarity in the use of different substrates. However, even within this compact group (Setophaga p. erithachorides, S. petechia, Protonotaria citrea, and L. peregrina) the foraging substrates used by L. peregrina differed from those used by S. p. erithachorides (Table 1B; Fig. 2D).
The use of foraging maneuvers showed a similar pattern than the use of foraging substrates. P. noveborascensis stand out from the other four species which group together (Table 1C; Fig. 2E). When P. noveborascensis was excluded from the analysis, L. peregrina differed in the use of foraging maneuvers with S. p. erithachorides (Fig. 2F; Table 1D). This indicated that P. noveborascensis used a set of substrates and foraging maneuvers that notably differed from the substrates and maneuvers used by the other four warbler species. On the contrary, S. p. erithachorides used a wider range of substrates and maneuvers than the other species (Fig. 2C-F).
Foraging substrates and foraging maneuvers- S. p. erithachorides: The foraging substrates used by S. p. erithachorides did not differ whether the migrant warblers were present or not (F = 1.26, P = 0.313). However, the used of foraging maneuvers differed between both periods (F = 3.55, P = 0.004). When migrants were present, S. p. erithachorides used more maneuvers, and slightly more homogeneously as indicated by cv values (cvpresent = 3.48, cvabsent = 3.60).
Warblers’ morphology: The morphology differed between groups of species. S. p. erithachorides, S. petechia, and L. peregrina did not differ in their morphology (Fig. 3). P. citrea and P. noveborascensis differed from the two Setophaga and L. peregrina, and P. noveborascensis differed from the other four species (Fig. 3).
Discusion
Behavioral ecology studies often provide relevant information on the factors underlying the coexistence of closely related species. In this study warblers exhibited foraging strategies that differed remarkably among species in a mangrove forest. There are two well-defined groups (Fig. 2C-F); one of such groups includes only a single species, the ground foraging Parkesia noveborascensis, which stands out from the rest of species. This is a species that forages primarily on the ground, gleaning for insects and other invertebrates on bare soil or in the litter. The other warblers form a more compact group (Supplementary Table 2). They primarily forage by gleaning prey from leaves and twigs, but there are some differences between S. p. erithachorides and L. peregrina. Although, both species forage mostly by gleaning, S. p. erithachorides glean 45% of its time on leaves and 46% of its time on twigs, while L. peregrina glean 80% of its time on leaves, making the foraging of this species different from the other species in the group (Fig. 2, Supplementary Table 3).
Morphology is usually associated with particular foraging strategies and microhabitat use in different groups of species (Brandl, et al., 1994, Fitzpatrick, 1985; Losos, 1990c; Moermond & Denslow, 1985; Norberg, 1994). Hence, species with similar morphologies, as a result of closely phylogenetic relatedness (or convergent evolution) tend to occupy similar microhabitats and use similar foraging strategies (Brandl, et al., 1994, Losos, 1990c). Within the studied warblers, the most distant species (i.e., P. noveboracensis) has the most discrepant morphology and foraging strategy (Lovette & Bermingham, 1999; Klein et al., 2004; Lovette et al., 2010). Protonotaria citrea and L. peregrina (= Vermivora peregrina) are, each one, placed in a different clade but both closer to the Setophaga (= Dendroica) clade than P. noveborascensis (Lovette et al., 2010). Protonotaria citrea differed morphologically from Setophaga species, but the morphology of Leiothlypis is similar to that of Setophaga spp. However, Protonotaria have a similar foraging strategy than both Setophaga species, despite their morphological differences, while the foraging pattern of L. peregrina differed at least from that of S. p. erithachorides, despite their high similarity in morphology. In the case of Setophaga, both taxa have similar morphology and similar foraging strategies. Therefore, although morphology associates with similar foraging strategies in this group of warblers, there are some subtle differences in foraging patterns likely determined by species specific foraging adaptations (e.g., preference for certain prey type) or other morphological features (e.g., wing loading) not considered in this study.
The foraging strategy of S. p. erithachorides changes when migrants arrive. The use of foraging substrates does not change but there was a tendency to use other foraging maneuvers (e.g., gleaning of the ground) or use some maneuvers more frequently (e.g., hanging, hovering) when migrants were present. Competition is usually advocated to explain changes in habitat use and foraging behavior, particularly when species interact with similar and abundant counterparts with similar morphology and foraging strategies (Bennett, 1980; Cody 1985; Diamond, 1978; MacArthur, 1958). However, other factors may usually explain the changes in habitat or foraging strategies attributed initially to interspecific competition (Morse, 1985; Strong, 1984; Wiens, 1989). For instance, the period of winter residence coincides with the period of minimal insect abundance in northwestern Costa Rica (Hespenheide, 1980; Janzen, 1980). This fact could be enough to change the foraging strategy of S. p. erithachorides during the wintering period of migratory warblers, if birds focus on other (or more) prey types. Thus, more generalist behavior is expected when resource availability decreases (Carpenter & MacMillen, 1976; Grant, 1993), but further evidence is required to support this hypothesis.
Differences and similarities in the foraging strategies of the five warbles species match the species’ morphology. This suggests that the foraging strategy of each species has been molded by different (or similar) adaptation processes along the evolution of each species or group. Therefore, species that have occupied the same adaptive landscape or are constrained by their recent ancestry-such as S. p. erithachorides and S. petechia (Chavarria-Pizarro et al., 2019)-are expected to exhibit more similar morphologies and foraging strategies. Our results provide little support for the niche partitioning hypothesis, as similar species (morphologically and/or phylogenetically) use the habitat similarly-contrary to the prediction that similar species would use the habitat differently. Competition cannot be entirely excluded, but it would be only one aspect, like predation and seasonal changes in resources, of the adaptive scape in which each species evolved.
Ethical statement: the authors declare that they all agree with this publication and made significant contributions; that there is no conflict of interest of any kind; and that we followed all pertinent ethical and legal procedures and requirements. All financial sources are fully and clearly stated in the acknowledgments section. A signed document has been filed in the journal archives.

