


 Inglés (pdf)
 Articulo en XML
 Referencias del artículo

 Traducción automática
 Enviar articulo por email
 Citado por SciELO
 Similares en
SciELO
 uBio

 Permalink


Introduction
Urban areas worldwide are expanding rapidly due to human population growth. Continuous urbanization transforms natural and rural environments, leading to the formation of urban centers (Aronson et al., 2015; Montgomery, 2008). Species abundance and diversity depend not only on the level of urbanization but also on the taxonomic group (Blair, 1996; Lewis et al., 2015; Lindenmayer et al., 2002). Urban centers often exhibit low species diversity due to altered biological composition and, consequently, altered ecological relationships between these species (Marzluff, 2001; Marzluff, 2017).
In tropical regions, the largest group of social bees are stingless bees (Apidae: Meliponini), with approximately 550 described species; they exhibit an eusocial lifestyle with perennial colonies (Grüter, 2020). Monitoring bee colonies facilitates long-term demographic studies, and the results of these studies can be applied in stingless beekeeping, known as “meliponiculture” (Grüter, 2020). Stingless bees are important pollinators and play crucial roles in ecosystem maintenance and food availability (Heard, 1999; Klein et al., 2018; Roubik, 2023; Slaa et al., 2006). Several stingless bee species have been shown to adapt very well to urban conditions (Roubik, 2023; Velez-Ruiz et al., 2013; Vieira et al., 2016). However, studies on the impact of urbanization on bee diversity and abundance are relatively rare but more important than ever due to rapidly increasing urbanization (Solano-Gutiérrez & Otárola, 2025). To maintain bee diversity and thus ecosystem services, including pollination, bee conservation is essential and can only be achieved by developing protection measures based on bee ecology and knowledge of bee distribution.
In Costa Rica, the Central Valley represents the largest urban settlement, including the capital city San José and other major cities, forming a metropolitan area inhabited by 60% of the country’s population (Madrigal-Solís et al., 2019; Muñoz et al., 2021). Costa Rica has 59 species of stingless bees (Moure et al., 2007), of which several are abundant in urbanized environments, especially when trees are abundant, but the species composition and dynamics have never been analyzed in an urban ecosystem in Central America.
In this study, we quantified the frequency and species richness of stingless bee nests in 2016 and 2022 on a university campus within an urbanized area. Additionally, bee host plants and nesting sites were documented providing information on strategies for survival in urban environments. We assessed whether bee diversity and abundance changed between 2016 and 2022; we calculated a bee nest survival rate and determined whether there was a turnover in species using a specific nest location. Thus, we identify host plant species and evaluate nesting location preferences: substrate and nesting height.
Materials and methods
Location: The study was conducted at the Rodrigo Facio Campus of the University of Costa Rica (UCR), which occupies approximately 97 hectares across three contiguous sites. The Campus is located in Montes de Oca, San José, Costa Rica (9°56’15”N 84°03’01”W; 1200 m a.s.l.). The climate is classified as tropical, with an annual mean precipitation of 1 868 mm (±358 SD) and an annual mean temperature of 20 °C (CIGEFI, 2025). The region’s dry season is from December to April, and the rainy season is between May and November (Sáenz et al., 2007).
The censuses considered only the site called Finca 1 (31 ha), the first one established in 1956, with the oldest buildings and trees. The other two campus sections experienced large disturbances (infrastructure development) at the time of the study, and their sampling was logistically unfeasible. The population of the campus is approximately 40 000 people (UCR, 2024). The sampled area has a high density of buildings and infrastructure (58 % impervious surfaces and 42 % natural, seminatural, or green areas); the area surrounding the campus is highly urbanized (Fig. 1).
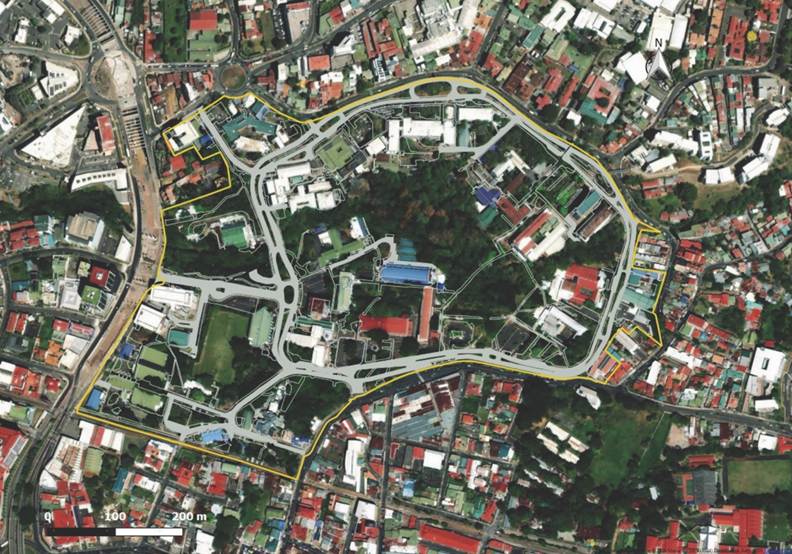
Fig. 1 Campus of the University of Costa Rica (only Finca 1 is shown) and the surrounding urban area of Montes de Oca, San José. The yellow line delineates the sampled area. Within this polygon, gray stripes represent roads, and white lines delineate trails, sidewalks, and parking lots. Source: OEPI, UCR; Bing aerial 2024, Microsoft Corporation.
The flora of the campus is diverse, with a variety of native versus introduced and wild versus planted trees, shrubs, and herbaceous plants, which are intensively managed. This flora provides a variety of nesting and foraging resources for wild bees. The campus center hosts two hectares of regenerated forest area.
Data acquisition and visualization: Data were collected in 2016 (September-December) and 2022 (December-March). The area was searched systematically for stingless bee colonies (active nests) on trees and man-made infrastructure. Every tree and every man-made element were visually examined from all sides, from the ground to the top. The campus area was run through several times by foot for each survey. In this context, “trees” include any section (internal or external) of living or dead trees, remnant tree trunks, palms, or bamboo. “Infrastructure” refers to anything man-made, such as walls, buildings or fences. Since no ground-nesting species have been reported on the campus in the past nine years of sampling, ground nests were excluded from searching. Each tree species hosting a nest was identified, and each nest was marked with coordinates using GPS (GPSmap® Garmin CSX60), with an average error of less than 2 meters. We analyzed tree species data only for 2022 because the trees used by bees in 2016 were also used in 2022.
In 2022, we first searched all preexisting nests based on the survey conducted in 2016, as well as every new location. The same search protocol was used for both samplings. The use of tags was avoided to prevent attracting the attention of users of the campus, which could negatively affect the nests. Finally, each colony was initially identified at the species level based on the nest entrance architecture and voucher specimen collected from each nest. Representative specimens were deposited at the Museum of Zoology (MZUCR) of the University of Costa Rica.
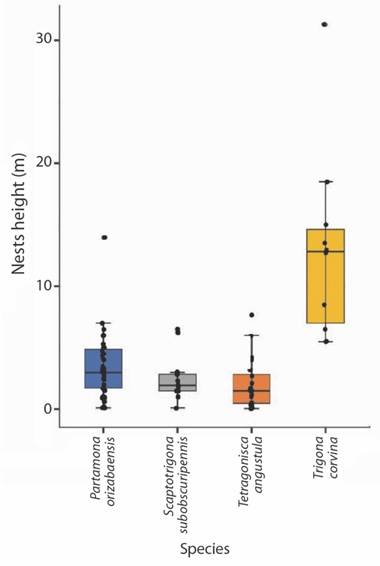
Additionally, we measured nest height to identify species-specific preferences in nest construction using a distance meter (Leica Disto™ D2). To identify species-specific differences in nest height, a Dunn (1964) Kruskal‒Wallis test was performed. Lestrimelitta mourei was excluded because of its low nest count (n = 2). The test was performed in R (https://www.R-project.org/; Version: 2022.02.0+443).
Results
Nest abundance and species diversity: In total, 68 stingless bee nests (2.13 nests/ha) were found on the Campus of the University of Costa Rica in 2016, and 86 (2.69 nests/ha) were found in 2022, representing a 26.5% increase in abundance. In both surveys, the same five different stingless bee species were found: Partamona orizabaensis (Strand, 1919), Tetragonisca angustula (Latreille, 1811), Scaptotrigona subobscuripennis (Schwarz, 1951), Trigona corvina (Cockerell, 1913), and Lestrimelitta mourei (Oliveira and Marchi, 2005). The abundance of four species increased over the six-year period (Table 1). Partamona orizabaensis was the most abundant species, comprising nearly half the nests found during both samplings, followed by Te. angustula. The cleptoparasitic L. mourei was the least abundant species, with only one nest in each sampling (Table 1). Nest survival was high, ≥ 56% for every species, except for L. mourei. Additionally, only one of the original nests was reoccupied by a different species; one S. subobscuripennis nest was formerly occupied by P. orizabaensis.
Table 1 Frequency and percentage of eusocial bee nests according to year on the Campus Rodrigo Facio of the University of Costa Rica and changes between censuses.
| Species | 2016 | 2022 | Increase in abundance (%) | Survival 2016-2022 (%) | |||
| Count | % | Count | % | ||||
| Partamona orizabaensis | 39 | 57.35 | 42 | 48.84 | 7.69 | 56.40 | |
| Tetragonisca angustula | 16 | 23.53 | 21 | 24.42 | 31.25 | 68.75 | |
| Scaptotrigona subobscuripennis | 6 | 8.82 | 12 | 13.95 | 100 | 83.30 | |
| Trigona corvina | 6 | 8.82 | 10 | 11.63 | 66.67 | 100 | |
| Lestrimelitta mourei | 1 | 1.47 | 1 | 1.16 | 0 | 0 | |
| Total | 68 | 100 | 86 | 100 | 26.47 | 64.70 | |
Nesting location preferences: With one exception, T. corvina, all species built nests in preexisting cavities in trees or man-made structures. In both surveys, most bee nests were found on trees (Fig. 2). Tetragonisca angustula and P. orizabaensis were the only stingless bees found nesting in infrastructure. The number of Te. angustula nests built on infrastructure doubled between the censuses, but those of P. orizabaensis decreased to one third.
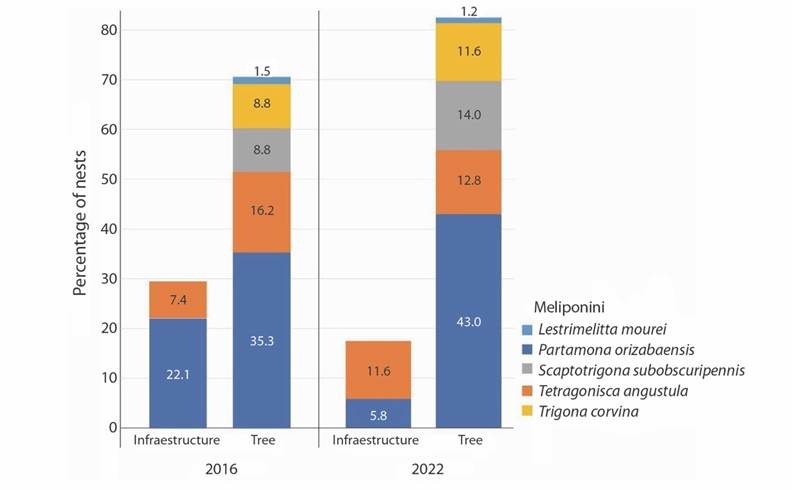
Fig. 2 Percentage of stingless bee nests per sampling year according to species and nesting substrate (infrastructure or tree) on the Campus Rodrigo Facio of the University of Costa Rica.
In 2022, bees inhabited 26 different tree species (Table 2). Among them, 32.4% of all nests were found on two native species of fig; Ficus jimenezii hosted the most nests, including all the bee species found in this census (Table 2). Furthermore, in Ficus costaricana, three different bee species were found (S. subobscuripennis, Te. angustula, and T. corvina). Taken together, Cupressus lusitanica and Spathodea campanulata, two introduced tree species, hosted approximately 22% of the nests (Table 2).
Table 2 Tree species used by stingless bees for nest construction, categorized by their origin.
| Family | Species | Status | Nest count | Percentage of nests per tree species |
| Moraceae | Ficus jimenezii | Native | 19 | 26.8 |
| Cupressaceae | Cupressus lusitanica | Introduced | 8 | 11.3 |
| Bignoniaceae | Spathodea campanulata | Introduced | 7 | 9.9 |
| Moraceae | Ficus costaricana | Native | 4 | 5.6 |
| Boraginaceae | Cordia eriostigma | Native | 3 | 4.2 |
| Myrtaceae | Melaleuca quinquenervia | Introduced | 3 | 4.2 |
| Arecaceae | Roystonea regia | Introduced | 2 | 2.8 |
| Bignoniaceae | Tabebuia rosea | Native | 2 | 2.8 |
| Poaceae | Bambusa sp. | Introduced | 2 | 2.8 |
| Cupressaceae | Chamaecyparis sp. | Introduced | 1 | 1.4 |
| Anacardiaceae | Mangifera indica | Introduced | 1 | 1.4 |
| Anacardiaceae | Tapirira mexicana | Native | 1 | 1.4 |
| Arecaceae | Elaeis guineensis | Introduced | 1 | 1.4 |
| Bignoniaceae | Jacaranda mimosifolia | Introduced | 1 | 1.4 |
| Casuarinaceae | Casuarina equisetifolia | Introduced | 1 | 1.4 |
| Clusiaceae | Garcinia mangostana | Introduced | 1 | 1.4 |
| Fabaceae | Cojoba arborea | Native | 1 | 1.4 |
| Fabaceae | Erythrina poeppigiana | Introduced | 1 | 1.4 |
| Lythraceae | Lagerstroemia speciosa | Introduced | 1 | 1.4 |
| Malvaceae | Ceiba pentandra | Native | 1 | 1.4 |
| Meliaceae | Cedrela odorata | Native | 1 | 1.4 |
| Moraceae | Ficus elastica | Introduced | 1 | 1.4 |
| Moraceae | Ficus sp. | Introduced | 1 | 1.4 |
| Myrtaceae | Eucalyptus sp. | Introduced | 1 | 1.4 |
| Sapindaceae | Cupania glabra | Native | 1 | 1.4 |
| Verbenaceae | Citharexylum donnell-smithii | Native | 1 | 1.4 |
| Dead trees | 4 | 5.6 | ||
| Total | 71 | 100 |
Partamona orizabaensis was found in 16 different tree species, of which most of the nests were built in F. jimenezii, S. campanulata, and C. lusitanica. This bee species also nests abundantly in human infrastructure (Fig. 2). Scaptotrigona subobscuripennis nests were evenly distributed among eight different tree species. The same distribution could be observed for Te. angustula, which was found with one nest each in seven different tree species, except in F. jimenezii, which had five nests. Trigona corvina nests were also distributed among five different tree species.
Nesting height: The average nesting height of all stingless bee nests found in this survey on the campus was 4.07 m above ground level. For pairwise comparisons, nests from L. mourei were excluded since only two nests were found. The height of the nests differed significantly between species (Kruskal‒Wallis test, χ2= 27.91, P < 0.001). The average nest height of T. corvina was 12.99 m, which was significantly higher than that of all the other species (Dunn test, P < 0.001). Average nest heights from P. orizabaensis, S. subobscuripennis and Te. angustula were 3.42 m, 2.55 m, and 2.10 m respectively, and did not differ significantly from each other (Dunn test P > 0.1; Fig. 3).
Discussion
Nest abundance and species diversity: The abundance and diversity of bee species depend on various biotic and abiotic factors. On the Rodrigo Facio campus of the University of Costa Rica, only five species of stingless bees were found. The key factors influencing nesting success in stingless bees include food source availability, nest site availability, and human alterations in the environment (Eltz et al., 2002; Grüter, 2020; Roubik, 2023). Urban areas typically lack sufficient food resources, which is a primary factor that reduces bee diversity (Wilson & Jamieson, 2019). The city of San José, where the study area is located, has reduced tree coverage and limited green spaces. These factors drastically reduce food availability and nesting spaces available for many bee species, further limiting their abundance and diversity (Solano-Gutiérrez & Otárola, 2025). In contrast, El Rodeo, a forest patch outside San José (800-1 000 msnm, 24 km W from the sampled area), which is surrounded by rural areas, hosts 13 genera of stingless bees, such as Cephalotrigona, Geotrigona, Melipona, Nannotrigona, Oxytrigona, Plebeia, Scaura, Tetragona, and Trigonisca, which are not present in the study area (M. F. Otárola, unpublished data).
Interestingly, the overall number of nests on the campus increased by >26% within six years. One of the most important factors for bee colonialization is the availability of nesting sites and food sources (Grüter, 2020). Here this corresponds to tree cavity availability and suitable infrastructure, such as walls with cavities (Hanson et al., 2021). Changes in vegetation and infrastructure cover between the censuses were minimal and should not have influenced the differences found (e.g., no new or dead nests were related to new buildings or cut trees).
A reasonable explanation for the increase in nest abundance could be the decreased presence of humans during the COVID-19 pandemic. The campus restricted student access from March 2020 until March 2022. The decrease in human-induced stress may have facilitated the increase in the number of nests.
The effect of disturbance can be calculated from the yearly mortality rate of stingless bees. Stingless bee nests often live for many years, while the longevity of workers is relatively short, one to several months, queens usually live between 1 and 3 years and sometimes even longer (Grüter, 2020). The annual mortality rates per species in the sampled area range from 0-7.9% (excluding L. mourei), and the highest values are from the species that use man-made cavities on infrastructure. The mortality rates reported here are lower than those reported in other studies. Eltz et al. (2002) monitored Trigona collina nests in undisturbed and managed forests in Borneo. They calculated a yearly nest mortality rate of 13.5-15.0%. Velez-Ruiz et al. (2013) estimated that the nest mortality rate of Te. angustula was lower than 10%. Slaa (2006) reported that colony survival depends on the bee species and location. This study found that the annual mortality rate of Te. angustula significantly depended on the habitat structure; colonies in deforested areas (not urbanized) lived three times longer than those inhabiting forests. Our sampling protocol would not detect cases in which a colony died but the nest was subsequently reoccupied by the same species, and mortality could be underestimated.
Nest substrate preference: Urban areas are structurally complex, offering many spaces for cavity-nesting bee species. Our findings suggest that trees are preferred for nest construction over artificial structures, with only two species using artificial structures for nesting (see Fig. 2). Partamona orizabaensis demonstrated the most generalist and adaptable nesting behavior, utilizing 16 tree species and various forms of infrastructure. This adaptability is related to its nest structure, as the species can build in semi open cavities and create exposed nests, allowing the colonization of locations unsuitable for other species. Tetragonisca angustula, the smallest bee in the survey with a small colony size, can use small-scale cavities in both trees and infrastructure. Tetragonisca angustula is particularly abundant in urbanized areas across the Neotropics (Aidar et al. 2013; Fierro et al. 2012; Velez-Ruiz et al. 2013; Vieira et al. 2016), with some studies indicating higher abundance in urban areas than in undisturbed environments (Fierro et al. 2012).
The other three stingless bee species have specific requirements that limit the availability of suitable nesting sites. Scaptotrigona subobscuripennis exclusively builds nests on living trees and requires large, well-formed cavities, which are less abundant. Trigona corvina constructs massive, exposed nests in canopy branches and do not require cavities. Undisturbed canopies are abundant at the campus site, suggesting that the number of T. corvina colonies will likely increase in the future, continuing the observed trend of a 67% increase in abundance during the sample period. Lestrimelitta mourei also requires well-formed cavities for nesting, but its biology as an obligatory cleptobiont limits its abundance, as this species is likely to maintain only small populations in this area.
Nesting height: There are no comparative data on nest-building heights between urban and undisturbed areas. The nests of T. corvina were the highest and largest among all the species observed. Trigona corvina nests are fully exposed in tree canopies, whereas other species typically expose only their nest entrance (Grüter et al., 2016). These nests can weigh up to 100 kg (Roubik & Moreno Patiño, 2009) and are particularly vulnerable to predators and disturbances, which may explain the highly aggressive behavior of T. corvina (Grüter, 2020) and their exceptionally high nesting height. In contrast, the tree cavities used by other species are located primarily in the lower parts of trees, leading to relatively lower nesting heights, indicating that nest-building height is influenced by nest architecture and the availability of suitable nesting sites in urbanized areas (Grüter et al., 2016).
Host‒plant interactions and their implications for conservation: In the 2022 survey, stingless bees used 23 different plant species for nest construction. Strangler figs (Ficus spp.) were the most important trees due to their growth habit. These trees begin as epiphytes, with their roots growing downward and encircling the host tree, eventually killing it (Schütt & Lang, 2004). The decomposing host tree leaves an empty space within the fig tree stem, creating ideal nesting sites for stingless bees (Grüter, 2020; Hanson et al., 2021). The utilization of figs in tropical urban areas could be a crucial strategy for providing natural nesting sites for eusocial bees. For instance, Ficus jimenezii hosted all the stingless bee species found on the campus. Ficus costaricana also harbored three species, but this species reaches smaller sizes than F. jimenezii, which is a probable reason for the lower number of colonies using this species. Introduced species, such as Spathodea campanulata and Cupressus lusitanica, harbored many nests due to their high number of cavities. However, each bee species utilizes a wide range of tree species, indicating that the availability of suitable cavities, rather than specific tree species, is critical for nesting.
The campus of the University of Costa Rica in San José was created on old pastures and coffee plantations and has been reforested since its foundation, allowing large and diverse trees to be present today, including large fig trees that require several decades to kill the host tree and eliminate its trunk. This landscape contrasts with the surrounding city, where few trees are present and most of them are small in size, precluding the existence of large natural cavities. Our results demonstrate that large stingless bee populations can develop in urban environments with complex tree coverage, especially if large trees are present. This information should guide management strategies that prioritize reforestation and the maintenance of large urban trees to support the establishment and maintenance of stingless bee colonies in urban environments. Combined with the ongoing planting of native ornamental plants that offer food resources, this can transform tropical cities into truly bee-friendly spaces.
Ethical statement: the authors declare that they all agree with this publication and made significant contributions; that there is no conflict of interest of any kind; and that we followed all pertinent ethical and legal procedures and requirements. All financial sources are fully and clearly stated in the acknowledgments section. A signed document has been filed in the journal archives.

