


 Inglés (pdf)
 Articulo en XML
 Referencias del artículo

 Traducción automática
 Enviar articulo por email
 Citado por SciELO
 Similares en
SciELO
 uBio

 Permalink


Introduction
Costa Rica is a small country in Central America, but with a varied topography, from coastal lowlands to high mountain ranges and volcanoes up to 3 800 m.a.s.l.. In this varied landscape there are numerous lakes and wetlands at all altitudes which harbor diverse crustacean fauna that is not yet well known in many groups. In 1984, Carmen Collado and coworkers published a first list of zooplankton from many sites in the country, as part of her master’s studies (Collado et al., 1984). It included a total of 67 species of Cladocera, Copepoda, Ostracoda and Rotifera. However, recent publications extended their list in Copepoda (Morales-Ramírez et al., 2014) and Rotifera (Kuczynska-Kippen & Ejsmont-Karabin, 2020). In a recent review of the literature on neotropical zooplankton for the region of Central America and the Caribbean, it was concluded that this microscopic fauna is still poorly known in the region, except for Guatemala, Costa Rica, and Nicaragua (Umaña-Villalobos et al., 2023). In this latter review, the number of zooplankton species reached a total of 190, with 27 species of Cladocera for Costa Rica. Nevertheless, studies have not been systematic enough to give a detailed picture of the richness and distribution of these groups.
Cladocera comprise a monophyletic group of microcrustaceans present in most continental waters. They are mainly part of the freshwater zooplankton; however, they are also found in the littoral and the benthos. Approximately 620 species are known for this group, but the real number might be from two to four-fold greater (Forró et al., 2008).
Cladocera are an important component in trophic webs in lakes and reservoirs, as they are preyed upon by many other species of fish, and therefore are indispensable for their growth and development (Gámez-Barrera et al., 2014). Knowledge on these groups is important, since freshwater habitats are under an increasing threat from different sources, such as pollution, drainage, and climate shifts, all which could cause their original faunal extinction and disappearance of the habitats (Ahmed et al., 2022; Grizzetti & Poikane, 2024). There is increasing concern about their state and preservation. All these groups could give useful information about key aspects of the situation of epicontinental freshwater habitats, which could help in planning sound management efforts to guarantee their recovery and conservation (Frolova, 2018; Green et al., 2005).
It is now clear that many widespread Cladocera species are, in reality, a species complex, composed of multiple local varieties which could be considered as separate species on their own, but not yet fully distinguishable among them unless using molecular information (Petrusek et al., 2003). However, it is necessary to increase the knowledge of the composition of local fauna using the most up-to-date taxonomic resolution, when possible. There are no taxonomic publications about Cladocera for Costa Rica, and their identification is performed utilizing keys for the United States, Mexico, and South America, in most cases. This situation leads to many gaps and doubts about their identity. As an example, there have been found several varieties of Daphnia in Costa Rica’s lakes and reservoirs that do not coincide with the descriptions in the available keys, and in some cases, there is confusion about whether they are the same species as described in the taxonomic guides. On the other hand, most of the information generated for this country is related to planktonic organisms, and there is a lack of information about littoral and benthic environments.
Despite all that, Cladocera diversity has been little studied in Costa Rica. This is the result of the taxonomic difficulties of the group and their small size, since their identification as a given species depends on the observation of detailed morphological descriptions of their thoracic limbs (Elías-Gutiérrez et al., 2008a). Furthermore, because it is a complicated group for correct identification, the work of specialists is required, but there are only few specialists devoted to Cladocera worldwide, and they are overloaded with material to be examined (Elías-Gutiérrez et al., 2008a; Frolova 2018). Nevertheless, there is information about the zooplankton of several lakes and reservoirs in Costa Rica, mainly from ecological studies performed in them and their zooplankton diversity. A total of 27 species of Cladocera in 16 genera and seven families have been observed so far (Umaña-Villalobos et al., 2023). The first report by Collado et al. (1984) gave a list of the organisms found in different freshwater habitats in Central America and the Caribbean. Their list includes a total of 22 Cladocera species. Haberyan et al. (1995) studied a total of 30 lakes in Costa Rica, and they report only six species of Cladocera. That same year, Umaña & Jiménez (1995) reported four species in lake Chato. On the other hand, Arenal Reservoir has been studied in more detail during several projects regarding its ecology, diversity, and monitoring, which allowed a more intensive study of its zooplankton. Umaña & Collado (1990) reported five species of Cladocera. Later, in a study of the trophic relationships in the plankton of the reservoir, Gavlas (2012) reported seven species of Cladocera in it.
The most common cladocerans in Costa Rican lakes belong the genus Daphnia O. F. Mueller, 1785, Bosmina Baird, 1845, Ceriodaphnia Dana, 1853, Moina Baird, 1850 and Diaphanosoma Fischer, 1850, which can be abundant in the zooplankton. However, there are also reports of poorly known species of the Chydoridae family, which dwell in the littoral of lakes and reservoirs, but have been little studied (Umaña-Villalobos et al., 2023). For this reason, in 2016, we started a study of cladocerans from different locations in Costa Rica, with an emphasis on littoral habitats, to increase knowledge, and the aim of this study is to report information on their diversity, distribution and new additions to Costa Rica’s Cladocera fauna.
Materials and methods
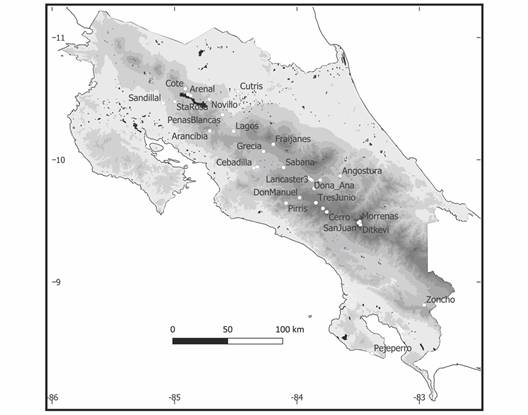
Samples were collected at different lentic sites in Costa Rica. Where it was possible, both littoral and open water column samples were taken. A total of 28 sites were visited from 2018 through 2020 for a total of 53 samples (Fig. 1, Appendix 1).
Sampling procedure: At each site, the water column and littoral zone were sampled. Water column samples were taken with a bongo plankton net with 64 µm pore size, performing a vertical or oblique tow from 1 m above the bottom up to the surface. Samplings in the littoral zone were taken using a smaller net, with the same pore size, tied to a handle that was passed through the vegetation. Samples were preserved in 90 % ethanol and brought to the laboratory at the Center for Research on Marine Sciences and Limnology (CIMAR), University of Costa Rica (UCR). Samples were first scanned at low magnification to withdraw individuals, which were kept in vials for later identification.
Sampling sites included in our study as well as in the literature reviewed were categorized according to their habitat type, and six habitat types were identified: Estuary, Lake Open Water, Lake Shore, Peatbog, Pond, and Reservoir. Species were assigned to those habitat types where they were collected, to examine the contribution of habitat type to the total diversity, and identify which species showed wider distributions.
Taxonomic identification: It was necessary to dissect every specimen for its identification, so that small structures that were needed according to taxonomic keys were observed. Wherever possible, 10 female specimens per species were examined, but in most cases, it was only possible to collect fewer specimens for each species. Most identifications were performed under the 100X immersion lens. When necessary, photographs were taken with an OMAX Toup View camera (24 megapixels) attached to the microscope. Identification was carried out utilizing the taxonomic keys of Elías-Gutiérrez et al. (2008b), Fernando (2002), Kotov & Štifter (2006), Maas (1998), Rogers et al. (2020) and Shiel (1995). We also consulted web pages devoted to Cladocera and biological diversity in general, such as gbif.org and itis.gov. Additional consultations were made with Cladocera experts.
Results
A total of 26 taxa of Cladocera were identified, of which 15 are new reports in Costa Rica (Table 1). With the new reports, the total number of Cladocera species for the country has increased up to 52 (Table 2). New records for Costa Rica are: Acantholeberis curvirostris (O. F. Müller, 1776), Acroperus TupinambaSinev & Elmoor-Loureiro, 2010, Biapertura ossiani (Sinev, 1998), Alonella dadayi Birge, 1910, Anthalona verrucosa (Sars, 1901), Camptocercus dadayi Stingelin, 1913, Chydorus dentifer Daday, 1905, Chydorus sphaericus (O. F. Müller, 1776), Ephemeroporus tridentatus (Bergamin, 1934), Flavalona iheringula (Sinev, 2004), Parvalona parva Daday, 1905, Simocephalus mirabilisOrlova-Bienkowskaja, 1998, Daphnia ambigua Scourfield, 1947, Leydigia striataBirabén, 1939 and Diaphananosoma brevireme Sars, 1901 (Table 1). There were several cases where it was not possible to assign an identification at the species level, including the following genera: Chydorus sp., Alona sp., Macrothrix sp., and Diaphanosoma sp., and a member of the subfamily Aloninae, which was not possible to identify to the genus level.
Considering the whole data set including data from literature, most species (63 %) were found at only one site, and only seven species were found in more than five sites (Appendix 2): Bosmina hagmanni Stingelin, 1904, Bosminopsis deitersi Richard, 1895, Ceriodaphnia cornuta Sars, 1855, Simocephalus serrulatus (Koch, 1841), Ilyocryptus spinifer Herrick, 1882, Moina cf. micrura Kurz, 1875, and Diaphanosoma spinulosum Herbst, 1975. Of these, Moina cf. micrura, which is reported from all continents, has been analyzed and demonstrated to be a species complex that is still poorly understood (Elías-Gutiérrez et al., 2019). Although the data are not necessarily representative of the diversity of lakes, ponds, reservoirs and other continental waters of Costa Rica, an analysis of the distribution of the fauna shows some tendencies. Most of the species occur in the open water of lakes (24 species), followed by ponds, where 16 species were found. In reservoirs, a total of 10 species were found. In estuaries, 13 species were reported (Appendix 3). It was only in lake Cote, which has a well-developed littoral zone, that vegetation sampling took place in this habitat, where 14 species were found. Seven species were found in the peatbog sampled in the Talamanca region. Six species were found in several habitat types: Ilyocryptus spinifer was found in five habitat types, Moinodaphnia macleaya (King, 1853), Diaphanosoma spinulosum, and Bosminopsis deitersi were found in four habitat types, and Simocephalus serrulatus, Moina cf. micrura, Ceriodaphnia cornuta and Daphnia laevis Birge, 1879 were collected in three habitat types. Eight species occurred in two habitat types, and the 39 remaining species were reported from just one habitat type. Among these latter, 11 species occurred in open water of lakes, eight on the lake shore, six in ponds, seven in estuaries, five in the peatbog and two in reservoirs. Similarity among habitat types was low, considering the few species that occurred in several habitat types. The most similar ones were Reservoirs, Open Lake waters and ponds.
Below, some morphological remarks are presented, regarding the new reported taxa from Costa Rica and their main ecological characteristics, based on the parthenogenetic females.
Cladocera Milne-Edwards, 1940 sensu
Family Acantholeberidae Smirnov, 1976
sensu (Dumont & Silva-Briano, 1998)
Genus Acantholeberis Lilljeborg, 1853
Acantholeberis curvirostris
(O. F. Müller, 1776) (Fig. 2)
Comments: Previously, it was considered as a member of the Macrothricidae Norman & Brady, 1867. Dumont & Silva-Briano (1998) observed some morphological characteristics in its appendices that confirmed separate evolution of Acantholeberis from the core-group of Macrothricidae. So, they proposed a new family, Acantholeberidae. For a long time, it was considered monotypic. In recent years, other new species from the neotropics have been described from Andean Colombia, Venezuela (Paggi & Herrera-Martinez, 2020) and lowlands in Brazil (Sousa et al., 2022).
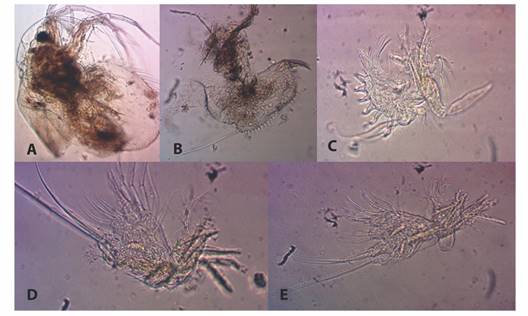
Fig. 2 Acantholeberis curvirsotris: A. habit, B. postabdomen. C. appendix 2, D. appendix, E. appendix.
What differentiates species in this genus is mainly their valve morphology and the proportion of some setae in the first, second and third appendices. A. curvirostris typically presents scrapers 5 and 6 of similar length on the second limb. Furthermore, the length of seta 6 of the exopodite on the third limb is shorter than half the length of seta 7 (Dumont & Silva-Briano, 1998; Hudec, 2010).
This species has been reported with a Holarctic distribution, mainly living in peatbogs there; this is the first report of species in latitudes below 23 °N. Typically, A. curvirsotris is found in mud and sediment, in muddy edges and small lakes, in pools and high-altitude paramos. It feeds by filtering the mud and bottom detritus. It is a sphagnolite and azidobiont species, strictly bound to oligo to mesotrophic waters, with a pH of 3.5 to 5.0 (Flößner, 2000). This coincides with the specimens found in Costa Rica, since this species was found in peatbogs in the Talamanca mountains.
Family Chydoridae
Dybowski & Grochowski, 1894
emend. Frey, 1967
Genus Acroperus Baird, 1843
Acroperus tupinamba
Comments: This is a Neotropical species which was described for the first time in Brazil (Sinev & Elmoor-Loureiro, 2010), where it is widely distributed and abundant. It occurs mainly amongst littoral vegetation in ponds, lakes, reservoirs, and streams. The species bears two spoon-like setae on the fourth limb exopodite, a unique morphological trait among Acroperus species. It can be distinguished by its short and broad postabdomen, with parallel sides, and long marginal setae on the valves. Head without a keel (Rogers et al., 2020; Sinev & Elmoor-Loureiro, 2010).
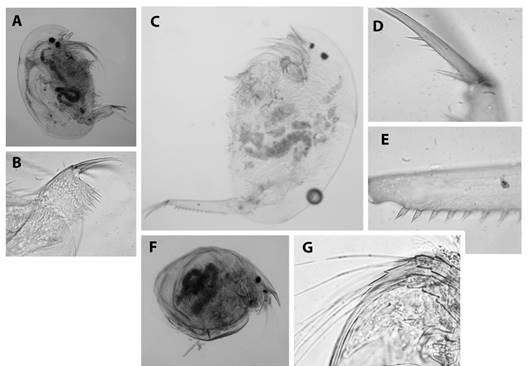
Fig. 3 Acroperus tupinamba, A. body, B. postabdomen. Camptocercus dadayi: C. body, D. postabdominal claw, E. postabdomen. Ephemeroporus tridentatus: F. body, G. detail of antenule.
Genus Biapertura Smirnov, 1971
emend.Sinev 2020
Biapertura ossiani (Sinev, 1998) (Fig. 4D)
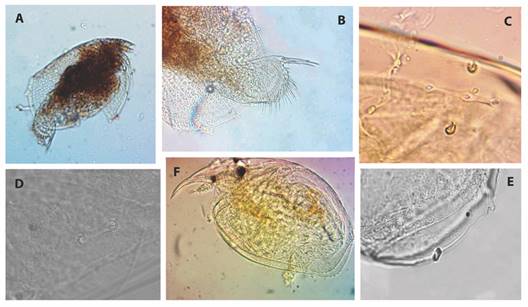
Fig. 4 Leydigia striata: A. body, B. postabdomen. Flavalona iheringula: C. pores. Biapertura ossiani: D. pores. Chydorus sphaericus: F. body. Chydorus dentifer: E. body.
Comments: B. ossiani is considered a sister species of the Palearctic Biapertura affinis (Leydig, 1860). These species clearly differ by their male morphology (eg. Sinev, 1998), but their females are not so obviously distinguishable (Sinev, 2009). According to this latter author, B. ossiani is the only species from the affinis group that is known in the Americas; however, recent data indicated the description of two subspecies: B. ossiani herricki is an invasive taxon in South Korea (Sinev, 2020). B. ossiani is a large cladoceran that reaches more than 1 mm in length. In the head there are two pores which are interconnected. The postabdomen is long, with a rounded distal postanal region, with 15 to 17 merged marginal spines. The basal spine is short. For more details, see Sinev (2020).
Genus Alonella G.O.Sars, 1862
Alonella dadayi Birge, 1910
Comments: The species has a long and curved rostrum, postabdomen narrow on the distal part and pre-anal angle markedly projected. This is mainly a neotropical species, distributed from the southern and eastern United States to the south of Brazil, where it is widely distributed and a common species (Sousa et al., 2020). These authors report the high variation in some morphological characters among populations and suggest that it might represent a species complex not yet elucidated. For more details, see (Sousa et al., 2020).
Genus Anthalona
Van Damme, Sinev & Dumont, 2011
Anthalona verrucosa (Sars, 1901) (Fig. 5)
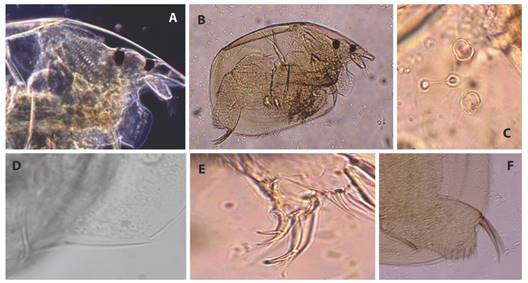
Fig. 5 Anthalona verrucosa: A. head, B. habit, C. pores 2, D. labrum, E. appendix I, F. Postabdomen.
Comments: Alona verrucosaSars, 1901 was transferred from the genus Alona Baird, 1843 (Anomopoda: Chydoridae: Aloninae) to Anthalona (Van Damme, Sinev & Dumont, 2011). The essential characteristic is the presence of two main pores in the head, and lateral pores with “Cosmarium” shape and sacs underneath them. It also has a short labrum with one or two denticles. The postabdomen is relatively short, deeply S-shaped, anal margin concave and postanal margin convex, with lateral fascicles not exceeding the level of marginal denticles; large proximal denticles on the inner distal lobe setae of the first limb. This species is very common and has a wide geographic distribution in the Neotropics (e.g. Paggi, 1975; Sars, 1901; Sinev & Hollwedel, 2002; Van Damme et al., 2011). It prefers basic to neutral environments but can tolerate mild acidity. For more details, see Van Damme et al. (2011).
Genus Camptocercus Baird, 1843
Camptocercus dadayi Stingelin, 1913
Comments: The main diagnostic characteristics of Camptocercus dadayi are the presence of a dorsal keel, a posteroventral margin of valves without denticles, a truncated rostrum, postabdomen, and narrowing of the basal spine at of the postabdominal claw with pecten presenting about ten spines (Sinev, 2015). This species occurs from the South-Eastern United States to South America (Sinev, 2018).
Genus Chydorus Leach, 1816
Chydorus dentifer Daday, 1905 (Fig. 4E)
Comments: In lateral view it has a globular outline. Body is high at the anterior half, narrowing posteriorly, and a straight posterior margin. The main characteristic is the presence of blunt denticles in the posteroventral margin of valves. It is also characterized by the presence of a large and oval labral keel. The postabdomen is elongated, four times longer than wide, with a long basal spine that reaches to the middle of the claw’s base. The three distal marginal denticles are stronger than the rest. This is a large Neotropical species (0.6-0.8 mm of length) (Elmoor-Loureiro, 2007; Smirnov, 1996), common in South America. It is rarely found, and little is known about its ecology, although it has been found at highly acidic sites (pH 4.2) in Lençóis and in Nhamundá River (Brazil), with a pH of 5.2 (Brandorff et al., 1982; Van Damme & Dumont, 2010).
Chydorus sphaericus (O.F.Müller, 1776) (Fig. 4F)
Comments: The species is recognized by its globular body, labral keel with distal portion elongated and triangular, postabdomen with preanal angle clearly prominent, postanal margin with distalmost portion slightly narrow armed with 7-8 denticles which have the base about 2.5-4.5 times shorter than the length itself (Sousa et al., 2024). There have been reported variations within this morphological scheme, but they are still inconclusive for separate species. Belyaeva & Taylor (2009) demonstrated the existence of at least seven species in the Holarctic region based on molecular evidence. Yet, it has been used as an indicator species due to its presumed ample resistance to environmental conditions, including low-pHs habitats (de Eyto, 2001). So, its presence in Costa Rica should be further analyzed as new information is gathered about their taxonomy; nevertheless, it is interesting to note that it was found in the peat bog we sampled. An invasion process should not be disregarded. This is a worldwide reported species; however, recent analyses point out that it should be considered a species complex, with numerous sibling species not yet described (Belyaeva & Taylor, 2009; Karabanov et al., 2022; Kotov et al., 2016).
Genus Ephemeroporus Frey, 1982
Ephemeroporus tridentatus (Bergamin, 1939) (Fig. 3F, Fig. 3G)
Comments: This is a Neotropical species, known from the south of Mexico, Venezuela, Colombia and Brazil (Barón-Rodríguez & Díaz, 2007; Elías-Gutiérrez et al., 2006; Elmoor-Loureiro, 1997). It is characterized by a lack of a dorsal keel in its carapace, labrum with three to four teeth, posteroventral margin of valves without denticles (Smirnov, 1996).
Genus Flavalona Sinev & Dumont, 2016
Flavalona iheringula (Sinev, 2004) (Fig. 4C)
Comments: It is a small (0.38-0.45 mm) oval-shaped chydorid which bears six limbs. It can be separated from the other Flavalona species by main head pores presenting narrow connections, lateral head pores circular with rounded sacs underneath them. This is a neotropical species, known from Colombia (Fuentes-Reinés et al., 2023) and Brazil (Brasil et al., 2019). It has been found more associated with sites with greater thalweg depth in streams in Brazil (Brasil et al., 2019).
Genus Leydigia Kurz, 1875
Leydigia striataBirabén, 1939
Comments: It is considered as a member of the acanthocercoides group by Kotov (2009) and Kotov et al. (2003), after studies which indicated insufficient data to confirm the description made by Birabén (1939) until revision based on the material from the type locality in Argentina. According to Rogers et al. (2020), its main diagnostic characteristic is a postabdominal claw basal spine rudimentary or absent. Postabdomen with maximum height not at midpoint, ventral margin straight. Leydigia c.f. striata also has a labral keel with lateral setulae, similar in length to anterior marginal setulae.
Genus ParvalonaVan Damme, Kotov & Dumont, 2005
Parvalona parva (Daday, 1905)
Comments: This species was formerly known as Leydigia parva, but Van Damme et al. (2005) considered it to belong to a different genus. It is a rare species that has been reported in South America, from Argentina to Colombia (Carvalho et al., 2024; Elmoor-Loureiro et al., 2009; Fuentés, 2015). It has a subovoid body, with a postabdomen conspicuously wide, armed with clusters of medium-sized marginal denticles (Van Damme et al., 2005).
Familia Daphniidae Straus, 1820
emend. Schoedler, 1858
Genus Daphnia O.F.Müller, 1785
Daphnia ambigua Scourfield, 1947 (Fig. 6)
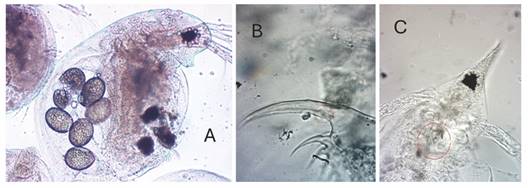
Comments: This species is common and widely distributed from North to South America and Europe (Benzie, 2005). Genetic data have revealed that there are several polygroups (Hebert et al., 2003), but it is still considered as a single species. It is small-sized Daphnia (up to 1 mm in length) that occurs in lakes and small ponds. It is characterized by its valve almost rounded, with a tail spine markedly shorter than valve length. The pecten on the postabdominal claws is armed with three groups of spines; the proximal group is clearly separated from the distal groups.
Genus Simocephalus Schoedler, 1858
Simocephalus mirabilis
Comments: This species occurs in the Nearctic and neotropical regions (Orlova-Bienkowskaja, 1998). It is characterized by a postabdominal claw with spines on the inner side and in the proximal part of the outer side. Basal part of the outer side with fine setulae which decrease in size evenly from base to the apex. Frontal part of head right-angled, with denticles, or very rarely without denticles. Posterior end of the carapace with a protruding rounded mound (Orlova-Bienkowskaja, 1998; Rogers et al., 2020).
Family Sididae Baird, 1850
Genus Diaphanosoma Fischer, 1850
Diaphanosoma breviremeSars, 1901
Comments: This is a neotropical species found from the south of Brazil to the south of Mexico and the United States (Elías-Gutiérrez et al., 2001; Korovchinsky, 2002; Sousa et al., 2009). The species can be recognized by the posteroventral margin of valves with groups formed by thin denticles increasing in length towards the posterior part of the valve (Sousa & Elmoor-Loureiro, 2021).
Discussion
Most of the new reports are from littoral habitats and the majority come from Lake Cote (61.5 %). This is the result of its diversity and abundance of aquatic plants along its shore. Only two species, Diaphananosoma brevireme and D. ambigua, are truly planktonic. This can be related to the fact that this habitat has been less studied in comparison to the open water habitat in most limnological studies.
It is also worth noting that more than 84% of the new records are species that belong to the family Chydoridae. This is one of the most diverse families within Cladocera, and most of its species dwell in littoral habitats (Fuentes-Reinés et al., 2021). The members of this family feed mostly on periphyton, and so their preference for the littoral zone might be related to the large quantities of organic detritus that are produced from decaying plants (Villabona-González et al., 2011). More studies are needed on their ecology since information is incomplete. It is also important to mention that some genera of this family can withstand extreme environmental conditions. Another example is the family Acantholeberidae, which is common in peatbogs, where pH is low. This family is being reported for the first time in Costa Rica and the whole Central American region (Paggi & Herrera-Martinez, 2020).
Although cladocerans are more diverse in the littoral zone, they have low population densities, which hinders their study. No one species was dominant, as is the case with planktonic species. Since it is only possible to capture a small number of individuals of each species, it becomes difficult to identify them properly to species level.
Four species that are reported for the first time in Costa Rica have not been reported in either Central America or the Caribbean, according to the account published recently by Umaña-Villalobos et al (2023). These species were Acantholeberis curvirostris, Acroperus tupinamba, Flavalona iheringula and Simocephalus mirabilis. Additionally, we update the nomenclature for six species reported earlier in the literature (Collado, 1983; Collado et al., 1984; Umaña-Villalobos & Aviles-Vargas, 2020), in accordance with the latest findings, especially in the genus Alona, family Chydoridae. These species are: Prendalona guttata (A. guttata), Prendalona barbulata (A. barbulata) (Sinev et al., 2023), Coronatella circufimbriata (A. circumfimbriata) (Sousa et al., 2015), Leberis davidi (A. davidi) (Sinev et al., 2005), Notoalona globulosa (Indialona globulosa) (Kotov et al., 2013), and Grimaldina freyi (G. brazzai) (Neretina & Kotov, 2017) in the family Macrothricidae.
It is possible that the actual diversity of benthic and littoral Cladocera is higher than is being reported here, since there are more wetlands and lakes that could not be included in our analysis here, especially those with wide areas covered with littoral vegetation, which are important as they house a rich fauna that is not fully studied yet (Biggs & Williams, 2024). It is also possible that some of the unidentified specimens represent species not yet described in the literature, since this group has been shown to present high levels of endemism and regional speciation, which has resulted in a high number of cryptic species even among species well-known worldwide (Belyaeva & Taylor, 2009). Besides, most species were found in just one site, with very restricted distributions, a sign of high beta diversity that may yet be discovered, hopefully in the not-too-distant future.
Ethical statement: the authors declare that they all agree with this publication and made significant contributions; that there is no conflict of interest of any kind; and that we followed all pertinent ethical and legal procedures and requirements. All financial sources are fully and clearly stated in the acknowledgments section. A signed document has been filed in the journal archives.
See supplementary material
a07v73s1-suppl1

