




 Inglês (pdf)
 Artigo em XML
 Referências do artigo

 Tradução automática
 Enviar este artigo por email
 Citado por SciELO
 Similares em
SciELO
 uBio

 Permalink

Introduction
Freshwater covers less than 1 % of the world’s surface area but harbors almost 10 % of all described species (Darwall et al., 2018; Dijkstra et al., 2014; Dudgeon et al., 2006; Mittermeier et al., 2010). Despite the indisputable importance of freshwater ecosystems in economic, cultural, aesthetic, scientific, and educational terms (see Dudgeon et al., 2006), we are facing a freshwater biodiversity crisis due to catastrophic declines in freshwater species and the degradation of these hydrological ecosystems (Darwall et al., 2018; Harrison et al., 2018; World Wildlife Fund (WWF), 2020). The Living Planet Report 2020 revealed a 94 % decline of the Living Planet Index for Latin America and the Caribbean, the most striking result observed in any region (WWF, 2020).
True or primary freshwater crabs (see Cumberlidge & Ng, 2009; Yeo et al., 2008) form with approximately 1 400 species an important part of the freshwater biodiversity in tropical and subtropical regions around the world (Yeo et al., 2008). The freshwater crab species diversity in the Neotropics - 311 species in three families (Trichodactylidae, Epiloboceridae and Pseudothelphusidae) - is only surpassed by that of east and southeastern Asia (Cumberlidge et al., 2014). According to the IUCN Red List conservation assessment, 34 % of the pseudothelphusids have an elevated risk of extinction, and 56 % of these species are too poorly known to assess (see Cumberlidge et al., 2014). Moreover, a recent assessment of the freshwater crabs in Colombia, which harbors the highest number of species in the Neotropics, revealed that pseudothelphusids are the most threatened freshwater crab species in this country (Acevedo-Alonso & Cumberlidge, 2021, Acevedo-Alonso & Cumberlidge, 2022). These data highlight the urgent need to obtain additional information about freshwater crab species inhabiting the Neotropics, especially about Pseudothelphusidae.
The Pseudothelphusidae is a very diverse family of primary freshwater crabs widely distributed throughout the Neotropical region, but the true extent of the geographic distribution of several species is poorly known because many of them occur in very remote areas with only a single or very few records available. For such species, therefore, all data relating to new occurrences are relevant as they are important for both taxonomic and biogeographic studies as well as for the development of regional and national assessments of the conservation status of the fauna. Here, we present new country records for three species of pseudothelphusid crabs: Phygiopilus acanthophallusSmalley, 1970 from Mexico and two from South American countries: Fredius stenolobusRodríguez & Suárez, 1994 from Guyana and Kunziana irengis (Pretzmann, 1971) from Brazil, as well as the confirmation of the occurrence of Raddaus mertensi (Bott, 1956) in Honduras. Considering that accurate information on the geographic occurrence and distribution of these species is scarce, here we discuss these new records and range extensions and highlight the importance of such data for the conservation assessment of freshwater crabs in the Neotropics.
Materials and methods
The new records are based on specimens that are preserved in ethanol 70 % and deposited at the following institutions: Forschungsinstitut und Naturmuseum Senckenberg (SMF), Frankfurt am Main, Germany; Instituto Nacional de Pesquisas da Amazônia (INPA), Manaus; Museu de Zoologia, Universidade de São Paulo (MZUSP), São Paulo, Brazil; and National Museum of Natural History, Smithsonian Institution (USNM), Washington D.C., U.S.A. Measurements of carapace are presented in millimeters; carapace width (cw) was measured across the carapace at its widest point, and carapace length (cl) was measured along the midline, from the frontal to the posterior carapace margin. The abbreviation “G1” refers to the male first gonopod and “coll.”/“colls.” to collector(s). The Portuguese word “igarapé” means creek or a small forest stream. The only locality without geographic coordinates originally informed in the label was tentatively georeferenced using Google Earth® software and these coordinates are given in brackets. Line drawings were made by CM using a Wild M8 (Wild, Heerbrugg, Switzerland) stereomicroscope equipped with a drawing tube attached, then scanned and edited in Adobe Photoshop® CS 2 software. The plates were mounted in CorelDraw® X3 software.
Results
Distributional data of four species of pseudothelphusid crabs, two of Raddausinae and two of Kingsleyinae, are presented for four Meso- and South American countries: P. acanthophallus in southeastern Mexico, R. mertensi in western Honduras, F. stenolobus in west-central Guyana, and K. irengis in northern Brazil.
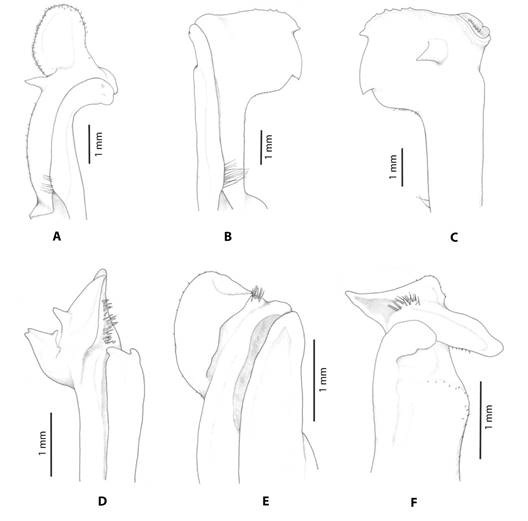
Fig. 1 Phrygiopilus acanthophallus, USNM 1180974, left male first gonopod, entire stem in mesial view (A); Raddaus mertensi, SMF 31690, right male first gonopod, distal portion in mesocaudal view (B) and laterocephalic view (C); Fredius stenolobus, MZUSP 24496, left male first gonopod, distal portion in mesocaudal view (D); Kunziana irengis, INPA 2565, left male first gonopod, distal portion in mesial view (E) and caudolateral view (F).
Raddausinae Álvarez, Ojeda, Souza-Carvalho, Villalobos, Magalhães, Wehrtmann
& Mantelatto, 2020 Phrygiopilus acanthophallusSmalley, 1970 (Fig. 1A)
Material examined: 2 males (cw 11.8, cl 8.0; cw 24.3, cl 15.2), 2 females (cw 19.5, cl 11.3; damaged), USNM 1180974, Mexico, Chiapas, near San Jose (San Jose de las Palmas, ~16°08’15”N 91°38’27”W), 28 miles ESE of Comitán (Comitán de Domínguez), 7-20.IV.1950, F.A. Pitelka coll.
Diagnosis: See Smalley (1970) and Rodriguez (1982).
Distribution: Guatemala (Alta Verapaz, Baja Verapaz, Zacapa) (Rodriguez, 1982; Smalley, 1970; Wehrtmann et al., 2016) and Mexico (present study).
Remarks: The identity of present specimens was determined by Martha R. Campos in June 1997, but this information has never been formally published (http://n2t.net/ark:/65665/3f6df1a83-408a-4140-8897-1ae4806b9974).
The G1 of the largest male from Chiapas, Mexico (USNM 1180974) resembles that of the holotype regarding its general morphology and, particularly, the proportions of the supra-apical process (Fig. 1A).
Raddaus mertensi (Bott, 1956)
Material examined: 1 male (cw 35.1, cl 22.5), 1 female (cw 24.5, cl 16.6), SMF 31690, Honduras, Ocotepeque, Guarin, cerro El Pital, 14°23.92’N 89°09.19’W, 14.V.1997, G. Köhler coll.
Diagnosis: See Rodriguez (1982).
Distribution: Guatemala (Chiquimula) (Wehrtmann et al., 2016), El Salvador (Santa Ana) (Bott, 1956), and Honduras (Ocotepeque) (Acevedo-Alonso & Cumberlidge, 2022; present study).
Remarks: The occurrence of R. mertensi in Honduras has already been reported by Acevedo-Alonso & Cumberlidge (2022) in a study on the conservation status of mountain species. However, these authors neither specified the distributional data of the specimen(s) nor reported the voucher material on which the record was based. The record presented herein confirms the occurrence of the species in the Ocotepeque department of Honduras.
The G1 of the specimen from Honduras is similar to that of the holotype except for the crenulation in the distal margin of the mesial process, which is slightly more pronounced in the Honduras specimen; furthermore, the small, rounded protuberance on the cephalic surface of the mesial process, which is present in the G1 of the holotype, is barely noticeable in the Honduras specimen (Fig. 1C).
Kingsleyinae Bott, 1970
Fredius stenolobusRodríguez & Suárez, 1994 (Fig. 1D)
Material examined: 1 male (cw 42.2, cl 28.3), MZUSP 24492, Guyana, Potaro-Siparuni, creek tributary of Kuribrong river, 05º27’N 59º31’W, 28.III.2011, F.C.T. Lima coll.
Diagnosis: See Rodríguez & Suárez (1994).
Distribution: Venezuela (Bolívar) (Magalhães & Pereira, 2003; Mora-Day & Blanco-Belmonte, 2008; Rodríguez & Suárez, 1994), Brazil (Roraima) (Zanetti et al., 2018), and Guyana (present study).
Remarks: The G1 of the present specimen is partially damaged, with a fissure at the base of the apical complex, just between the mesial process and the cephalic spine (Fig. 1D). Even so, it can be seen that the G1 morphology of the Guyana specimen is very similar to that of specimens from the Orinoco (see Rodríguez & Campos, 1998: 766, fig. 2A, B) and Amazon basins (see Zanetti et al., 2018: 4, fig. 1G). The only noticeable difference is in the G1 marginal process: in the present specimen, there is a small subdistal concavity whereas this concavity is very shallow in the specimen from the Amazon basin and indistinct in the specimen from the Orinoco basin.
Kunziana irengis (Pretzmann, 1971)
Material examined. 1 male (cw 23.0, cl 15.3), 1 female (soft carapace), MZUSP 45521, Brazil, Roraima, Uiramutã, Serra do Sol, Parque Nacional do Monte Roraima (= Mount Roraima National Park), igarapé Caramambai, near the bridge to the community Caramambatai, 05º07’58.8”N 60º35’08.8”W, 1005 m elev., collected with dip net, captured while copulating, 10.XII.2019, J. Zuanon, G.T. Vilara and R. Boldrini colls.; 1 male (cw 13.8, cl 8.4) 1 female (cw 19.5, cl 12.5), MZUSP 45522, Brazil, Roraima, Uiramutã, Serra do Sol, Parque Nacional do Monte Roraima (= Mount Roraima National Park), unnamed 2nd/3rd order stream, on the trail to the Ingarikó farm, 05º06’52.1”N 60º36’34.0”W, 1003 m elev., 05.XII.2019, J. Zuanon and D.A. Bastos colls.; 2 males (cw 20.0, cl 14.0; cw 21.3, cl 14.3) 1 female (cw 15.0, cl 10.5), CCDB 7811, Brazil, Roraima, Uiramutã, Serra do Sol, Parque Nacional do Monte Roraima (= Mount Roraima National Park), unnamed 3rd order stream, 05º07’07.5”N 60º36’21.0”W, 1043 m elev., 30.XI.2019, J. Zuanon and D.A. Bastos colls.; 1 male (cw 30.5, cl 19.7) 2 females (cw 23.3, cl 15.4; cw 30.3, cl 19.2), INPA 2565, Brazil, Roraima, Uiramutã, Serra do Sol, Parque Nacional do Monte Roraima (= Mount Roraima National Park), 05º07’36.2”N 60º35’36.7”W, 1008 m elev., 29.XI.2019, J. Zuanon and D.A. Bastos colls.; 1 female (cw 22.8, cl 16.2), INPA 2566, Brazil, Roraima, Uiramutã, Serra do Sol, Parque Nacional do Monte Roraima (= Mount Roraima National Park), unnamed 1st order stream, at the beginning of the trail to the Ingarikó farm, 05º07’37.7”N 60º35’58.6”W, ~1000 m elev., 30.XI.2019, J. Zuanon and D.A. Bastos colls.; 2 females (cw 22.6, cl 15.1; cw 22.7, cl 15.7), INPA 2567, Brazil, Roraima, Uiramutã, Serra do Sol, Parque Nacional do Monte Roraima (= Mount Roraima National Park), igarapé Sokopi (3nd/4th order stream), 05º07’27.7”N 60º35’49.3”W, 1005 m elev., 01.XII.2019, J. Zuanon and D.A. Bastos colls.
Diagnosis: See Magalhães et al. (2009).
Distribution. Guyana (Potaro-Siparuni) (Magalhães et al., 2009; Pretzmann, 1971) and Brazil (Roraima) (present study).
Remarks. The monospecific genus Kunziana is characterized by a very unusual G1 morphology in which the apical processes exhibit a combined strong twist in cephalic direction with a longitudinal bending towards the basal portion of the stem, causing the apical field of spines to face downwards (Magalhães et al., 2009: 42, fig. 1E-I). Such peculiar morphology can also be seen in the G1 of the Brazilian specimen of K. irengis examined herein, which, however, exhibits a slightly more developed patch of apical spinules on the distal portion of the caudal surface, and the apical plate is not so distinctly bilobed (Fig. 1F). These small differences could be attributed to the different sizes of the specimens examined or intraspecific variability.
Discussion
Species distribution: This is the first published record of P. acanthophallus from Mexico. The species was previously known only from Guatemala, in the departments of Alta Verapaz (Rodriguez, 1982; Smalley, 1970) and Zacapa (Wehrtmann et al., 2016), from the Caribbean Sea drainage area. The location of the present record in the department of Chiapas is located in the upper-median portion of the Usumacinta River basin, which empties into the Gulf of Mexico. The species, therefore, has a distribution that encompasses river systems draining into two versants. This new occurrence in Chiapas, near the border with Guatemala, also suggests that the species must have a wider distribution in northwestern Guatemala, since it would also be expected to occur in the upper portion of the Usumacinta River basin.
Documented records of R. mertensi were so far available only from its type locality, the Department of Santa Ana, in northwestern El Salvador (Bott, 1956) and from the Department of Chiquimula, eastern Guatemala, in the Pacific versant (Wehrtmann et al., 2016). Although the occurrence of the species has already been mentioned from Honduras (Acevedo-Alonso & Cumberlidge, 2022), this is the first documented record from the country, and such occurrence is not unexpected since the three known occurrences of the species are situated relatively close to each other in the region where the borders of the three countries converge, all in aquatic systems of the Pacific drainage.
Fredius stenolobus had already been recorded from the Caroni and Caura River basins in the state of Bolívar, Venezuela (Magalhães & Pereira, 2003; Mora-Day & Blanco-Belmonte, 2008; Rodríguez & Suárez, 1994), which are part of the Orinoco River basin, and from the Branco River basin in the state of Roraima, Brazil (Zanetti et al., 2018), an affluent of the Negro River, one of the main northern tributaries of the Amazon basin. Its occurrence in the Kuribrong River, an affluent of the Potaro River, which is part of the Essequibo River basin in west-central Guyana, is the first record of the species from this country. The present new record, therefore, reveals that F. stenolobus has a distribution that covers three different river basins draining the Guayana Shield region in northern South America.
Kunziana irengis has been originally found in the Guyanase side of the Maú/Ireng River basin (Magalhães et al., 2009; Pretzmann, 1971), the river that delineates the border between western Guyana and Brazil. The present record in creeks that are tributaries of the Contigo River (tributary of the Surumu → Tacutu → Branco → Negro → Amazon Rivers) confirms that it also occurs in Brazilian territory, as suggested by Magalhães et al. (2009). Both the Contigo River and the Maú/Ireng River, which also flows into the Tacutu River, are some of the northernmost tributaries of the Amazon basin. Although the known occurrences of the species in Guyanese territory are located on the southern flank of the Wokomung Massif, whose streams drain into the Maú/Ireng River basin, Magalhães et al. (2009) did not rule out the possibility that the species is also present in the Essequibo River basin, in streams that form the headwaters of the Potaro River in the northern portion of the aforementioned massif.
The presence of common elements of the aquatic fauna between the Essequibo and Branco River basins, as it is the case of F. stenolobus and K. irengis reported herein, as well as for other species of pseudothelphusid crabs (Mantelatto et al., 2022), can be understood in the context of the hydrogeomorphologic complex history of the region. This region was drained by the Proto-Berbice River basin that flew during Late Cretaceous to Early Quaternary from the southwest of the state of Roraima to the northeast of present-day Guyana. Tectonic and climatic events during the Plio-Pleistocene, however, promoted a rearrangement of the basin, especially the southward reversion of the Branco River and its entire northern catchment area, including the Maú/Ireng river drainage, into the Amazon basin, with a still existing connection area, the Rupununi Portal, a wetland region between the Tacutu and upper Essequibo rivers (Cremon et al., 2016; Ferreira et al., 2007; Lujan & Armbruster, 2011; Schaefer & Vale, 1999).
Conservation assessment: The IUCN global conservation assessment carried out in 2008 contains information only for three of the four species treated in this contribution: P. acanthophallus and R. mertensi were listed as “Vulnerable”, while F. stenolobus was classified as “Least Concern”. The fourth species, K. irengis, was not included in the 2008 IUCN global assessment, since it was considered as incertae sedis and as a non-valid species (C. Magalhães, personal observation, Sept. 2007). Only after this assessment, Magalhães et al. (2009) confirmed Kunziana as a valid genus and redescribed K. irengis. In the case of the three freshwater crab species included in the IUCN conservation assessment, all of them are lacking information about population size, population trends, and abundance. Moreover, their assessment was based on only three (R. mertensi and F. stenolobus) or four (P. acanthophallus) locations. In all three cases, the results of our study not only add new geographical reports/locations, but also include a new country previously not recorded for the species. Such information is important since it is the basis for the calculation of two evaluation criteria (Extent of occurrence and Area of occupancy) used for the assessment of the IUCN categories (International Union for Conservation of Nature (IUCN), 2012). Moreover, regular updating of the data is essential, as shown by the example of Colombia, the country with the highest number of freshwater crab in the Neotropics: between the first (2008) and the latest (2018) assessment, the percentage of threatened species in Colombia showed a dramatic increase from 26 % in 2008, to 34 % in 2015, to 62 % in 2018 (Acevedo-Alonso & Cumberlidge, 2021). Therefore, additional studies are constantly necessary not only to update and expand our knowledge about the different freshwater crab species but also to broaden and improve the information about threats affecting these macroinvertebrates.
A relatively high number of data-deficient species could lead to underestimations of the numbers of threatened freshwater species (Cumberlidge et al., 2014). In the case of K. irengis, this species has not even been assessed yet and only few specimens have been collected so far. The limited information available about the habitat of this species indicates that it occurs in clean rocky mountain streams with elevations ranging from 1 077 to 1 485 m (Magalhães et al., 2009). Just as in Colombia (see Acevedo-Alonso & Cumberlidge, 2021; Acevedo-Alonso & Cumberlidge, 2022), these montane environments might be threatened by increasing rates of deforestation, pollution, and human population growth. Serra do Sol, in the setentrional region of the state of Roraima, Brazil, is a mountainous region covered by savannah and forest situated within the Raposa-Serra do Sol Indigenous Land inhabited by indigenous people from several ethnic groups, an area that has experienced intense political conflicts between developers and the native population due to the region’s mineral, agricultural, and tourist potential (Lauriola, 2003; Sartori & Bethonico, 2018). Therefore, there is an urgent need to obtain additional information about K. irengis and to identify current threats to its habitat to develop adequate conservation measures for this species.
Although these new records only slightly expand the geographic distribution areas of these four Pseudothelphusidae freshwater crab species, they provide relevant new data for taxonomic and biogeographic studies, as well as for the development of better regional and national assessments of the conservation status of the aquatic fauna.
Ethical statement: the authors declare that they all agree with this publication and made significant contributions; that there is no conflict of interest of any kind; and that we followed all pertinent ethical and legal procedures and requirements. All financial sources are fully and clearly stated in the acknowledgments section. A signed document has been filed in the journal archives.

