


 Inglés (pdf)
 Articulo en XML
 Referencias del artículo

 Traducción automática
 Enviar articulo por email
 Citado por SciELO
 Similares en
SciELO
 uBio

 Permalink


Introduction
Leaves are among the most plastic organs in plants (Bradshaw, 2006; Kidner & Umbreen 2010; Nicotra et al., 2010; Reich et al., 1997; Wright et al., 2004; Wright et al., 2017), with their morphology, anatomy, and function reflecting adaptations to environmental gradients at the whole-plant level (Givnish, 1979; Reich et al., 1997; Sultan, 1987; Wright et al., 2004, Wright et al., 2017). While leaf structure is shaped by phylogeny (Givnish, 1987; Hay, 2019; Klingenberg et al., 2012), plants also show considerable leaf phenotypic plasticity within a species in response to environmental gradients (e.g., Martín-Sánchez et al., 2024). According to the functional convergence hypothesis, selective pressures-such as light, nutrient availability, and herbivory-converge on the leaf (Meinzer, 2003), making leaf structure a useful proxy for assessing whole-plant resource allocation strategies and adaptations to environmental changes (Pierce et al., 2022). This justifies efforts to identify integrative functional traits that connect leaf structure to whole-plant performance, from individual plants to ecosystems (de Bello et al., 2010; Díaz et al., 2016; Funk et al., 2017; Reich et al., 1997; Wright et al., 2004).
Key environmental factors such as nutrient distribution, temperature, water availability, and light influence resource allocation and plant function, impacting leaf structure (Nicotra et al., 2010). Leaf structure further determines energy absorption, affecting the leaf energy balance (Michaletz et al., 2015; Nobel, 1999). Features like boundary layer thickness and heat exchange can buffer leaves against environmental fluctuations (Nobel, 1999). For instance, small, narrow, and highly dissected leaves have a thinner boundary layer and higher heat dissipation capacity through convection compared to larger, entire leaves (Givnish, 1979; Vogel, 2009). In dry ecosystems, sun-exposed leaves are often smaller and more dissected, with greater lobulation and higher stomatal density than shade leaves, which experience more stable thermal conditions (Vogel, 2009). Increased lobulation supports heat dissipation more effectively than angling leaves to reduce light absorption (Vogel, 2009). Species with pinnately compound leaves can dissipate heat efficiently and lose individual leaflets rather than entire blades (Balding & Cunningham, 1976). The diversity in leaf size, shape, spatial arrangement, phenology, and heterophylly demonstrates the adaptive strategies that align leaf structure with fluctuating environmental conditions.
Plant functional traits serve as indicators of ecological and life-history strategies (Westoby et al., 2002), encompassing morphological, biochemical, physiological, structural, and phenological traits that influence performance and fitness (Cornelissen et al., 2003). Specific leaf area (SLA), which represents the fresh leaf area per unit dry mass, is a fundamental functional trait linking leaf quality to structure and function (Reich et al., 1998; Reich et al., 2003; Wright et al., 2004). SLA correlates with photosynthetic rate, nitrogen content, leaf lifespan, quantity and quality of defenses, and growth rate, reflecting trade-offs between light absorption and leaf construction costs, and thus, it influences overall plant performance and fitness (Reich et al., 1997). SLA is determined by internal leaf anatomy, tissue density, and chemical properties (Poorter et al., 2014; Villar et al., 2013), as well as by whole-plant allocation strategies (Pierce et al., 2022). Since SLA measures the cost of light interception at the leaf level, it also affects leaf energy balance and can serve as a proxy for acclimation to sun and shade environments over a leaf’s lifetime (Rozendaal et al., 2006).
The genus Monstera, known for high leaf heteroblasty (Andrade et al., 2008; Madison, 1977), includes nomadic vines (Zotz, 2013) that thrive on a range of substrates, such as trees and rocks. Monstera deliciosa Liebm. adapts to diverse light conditions, from sun-exposed canopy sites to shaded understories. In the shade, leaves tend to be smaller, with shorter petioles, and reduced fenestration and lobulation compared to those in well-lit environments (pers. obs). A mature M. deliciosa crown may have both sun-exposed and shaded leaves, with phenotypic adjustments likely following light availability. Leaf fenestration, along with dissection or lobulation, can be considered an environmentally influenced trait (sensu Muir, 2013) as multiple environmental factors shape its adaptive effects along light gradients.
This study examines the morphological and structural differences between sun and shade leaves of M. deliciosa, focusing on fenestration and lobulation. We predict (a) that mature sun and shade leaves will differ in fenestrated area and lobulation ratio (leaf perimeter relative to the square of effective area, excluding fenestrations). Highly fenestrated, dissected leaves may dissipate heat effectively under sun (Nicotra et al., 2008). We also anticipate (b) that sun leaves will have higher stomatal density and lower SLA than shade leaves, adapting to higher radiation and wind exposure with increased transpiration for cooling and a thicker, more robust leaf structure. Overall, we expect sun leaves to be smaller, more dissected and lobulated, with higher stomatal density and lower SLA compared to shade leaves.
Understanding the relationship between leaf structure and light gradients addresses a key question in plant physiology: adaptation in structure and function to distinct environments. This exploratory study aims to inspire future research on the role of fenestration and lobulation in Monstera species with diverse leaf morphologies.
Materials and methods
Site description: Data collection was conducted in San Pedro de Montes de Oca, San José, at the campus of the University of Costa Rica (UCR, 9°56’09.1” N & 84°03’02.9” W, 1 200 m.a.s.l.). The site is in the Central Valley, and the life zone classifies a tropical and premontane rainforest (Holdridge & Grenke, 1971). The average annual rainfall is 1 700 mm, and the average annual temperature is 22 °C (Herrera & Gómez, 1993).
Study species: The genus Monstera has 35 species in Costa Rica (Cedeño-Fonseca et al., 2022). The species M. deliciosa Liebm. (Araceae) is one of the most cultivated ornamental plants in the world (Cedeño-Fonseca et al., 2022; Madison, 1977). It is distributed from Mexico to Guatemala. It was introduced in Costa Rica, where it can be found from 400-2 000 m.a.s.l. (Grayum, 2004). The growth habit is hemiepiphytic or epiphytic scandent. Seedlings start on the ground and then colonize a vertical substrate, displaying small, entire leaves. The rhizomatous stem produces adventitious roots, enabling the plant to anchor itself to various substrates, including rocks and trees. The stem can lose contact with the ground but sends feeder roots down. This pattern of habitat colonization (starting life on the ground, then colonizing the canopy while maintaining a root connection on the ground) fits the definition of a nomadic vine (Sperotto et al., 2020; Zotz, 2013). The leaves experience a wide range of light gradients, from the understory to the canopy, as the plant colonizes different light environments, from highly shaded to highly exposed sites. In M. deliciosa, leaf development is highly plastic and seems associated with plant age and light conditions. For instance, in reproductive plants the leaves usually maintain a regular phenotype in terms of size and number of fenestrations, although in the highlands M. deliciosa may develop smaller leaves (Cedeño-Fonseca et al., 2020). The adult leaves of a mature plant have very deep lobes (6 to 12 lobes per leaf) and over 101 fenestrations, although the number of fenestrations is usually very regular (Cedeño-Fonseca et al., 2020).
Leaf selection according to distinct conditions of sun and shade: We selected M. deliciosa plants under distinctively different high light and deep shade conditions during September, October, and November 2022. The light environments of sun and shade were chosen to maximize light differences (i.e., sun leaves were clearly exposed to high light, and shade leaves were chosen below several layers of sun leaves). We chose only one mature, fully expanded leaf per plant and per light environment, in widely distributed M. deliciosa patches to make sure that leaves belong to different individuals. In total, we measured 20 leaves (one per patch), 10 for each light condition.
Quantification of leaf morphology and structure: Each sampled leaf was photographed in situ, with a large piece of white cloth placed behind it to enhance contrast. To ensure accurate measurements, the leaf surface was kept as flat as possible, and a 50 cm ruler was included in the frame for scale. Using ImageJ software (Schneider et al., 2012), we measured the total leaf area (including fenestrations), the fenestrated area, the effective leaf area (excluding fenestrations), and the leaf perimeter based on these photographs. Leaf length was measured directly from the base of the leaf blade to the tip using a measuring tape. Leaf width was determined by measuring from the tip of the sixth lobe on the left side of the leaf blade (starting from the base) to the tip of the sixth lobe on the right side. The fenestration ratio was calculated as the fenestrated area divided by the total leaf area. The lobulation ratio, equivalent to the leaf dissection index (Kincaid & Schneider, 1983), was determined by dividing the leaf perimeter by the square of the effective leaf area. We separated lobes from fenestrations; but we recognize that lobes begin as fenestrations by breaking through the leaf margin and thus forming the lobes (medium to small fenestrations remained within the leaf margin). This was an arbitrary distinction, but the purpose was to quantify leaf lobulation separated from the fenestration within the leaf margin. The length of the leaf petiole was measured from the point of petiole insertion on the stem to the beginning of the leaf blade.
Specific leaf area (SLA): SLA (cm2/g) is defined as the ratio of fresh leaf area to dry weight (Poorter et al., 2009). A section of fresh leaf area of 12.5 cm2 was obtained from the right side of every leaf near the central vein. The dry weight of this leaf section was measured after placing it in an oven at 60 oC for 3 days or until constant weight. Leaf mass was measured using a PRACTUM224-1S analytical scale.
Stomatal density: We took a 12.5 cm2 leaf segment from the middle of the central vein and at the end of the left lobe (abaxial surface) and reported stomatal density (SD) as the number of stomata (n stomata/mm2) within an area of 3 mm2 at a magnification of 100x under a light microscope using an imprint of a dried layer of clear nail polish.
Statistical analysis
Correlation structure of leaf morphological traits: We examined the relationships among nine traits describing leaf morphology and degree of leaf lobulation (Table 1). First, we calculated the Pearson correlation coefficients for these traits (Fig. 1) and then used principal component analysis (PCA) to summarize the correlation structure. From the 11 variables listed in Table 1, we selected nine: total leaf area was excluded due to redundancy with effective leaf area (correlation coefficient of 0.99), and fenestration ratio was excluded as it showed a high correlation (0.88) with fenestrated area, leaving only the fenestrated area. The variables entering the PCA were ln-transformed and centered to remove artifacts caused by scale and different units of measurement.
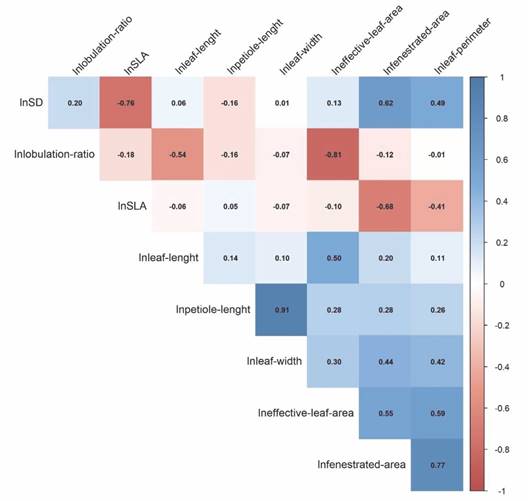
Fig. 1 Correlation matrix of nine ln-transformed morphological traits in 20 leaves of Monstera deliciosa. Values correspond to the Pearson correlation coefficient for each variable combination. SD = stomatal density, SLA = specific leaf area.
Leaf shape and morphology were summarized by the scores of the first three principal components (eigenvalues > 1, 82.88 % of the total variation), which were derived from the nine selected traits. To assess differences in these principal component scores between light conditions (sun and shade), we performed one-way MANOVA (Quinn & Keough, 2002). Following a significant MANOVA result, we conducted one-way ANOVAs on individual variables as post hoc tests to detect specific differences between sun and shade leaves. All analyses were performed in R, using the PerformanceAnalytics, factoextra, and FactoMineR packages.
Results
Differences between sun and shade leaves were evident in the magnitude of effective leaf area, fenestrated area (4.74 % of the effective leaf area in sun leaves and 1.88 % in shade leaves), fenestration ratio, leaf perimeter, and stomatal density. All these variables had higher magnitude in sun leaves, but SLA was higher in shade leaves (Table 1). Positive correlations were observed among fenestrated area, fenestration ratio, leaf perimeter, and stomatal density. The strongest positive correlation was between petiole length and leaf width, followed by the correlation between stomatal density and fenestrated area. The strongest negative correlation was found between lobulation ratio and effective leaf area (Fig. 1).
Table 1 Leaf morphological traits measured in Monstera deliciosa on the campus of the University of Costa Rica, San Pedro, Costa Rica, under sun and shade conditions.
| Leaf trait | Sun leaves | Shade leaves |
| Petiole length (cm) | 50.28 (4.43) | 52.22 (3.51) |
| Leaf width (cm) | 50.39 (5.11) | 48.35 (3.14) |
| Leaf length (cm) | 52.70 (4.58) | 49.80 (3.27) |
| Total leaf area (cm2) | 1 598 (105.53) | 1 500 (140.36) |
| Effective leaf area (cm2) | 1 522.18 (100.64) | 1 471.85 (132.78) |
| Fenestrated area (cm2) | 75.81 (9.81) | 28.14 (8.22) |
| Fenestration ratio | 0.046 (0.005) | 0.016 (0.003) |
| Leaf perimeter (cm) | 809.84 (47.27) | 659.28 (56.97) |
| Lobulation ratio (dissection index) | 0.00037 (0.000035) | 0.00033 (0.000034) |
| Stomatal density, stomata/cm2 | 17.53 (0-64) | 10.83 (0.56) |
| SLA (cm2/g) | 84.78 (2.14) | 132.16 (4.36) |
Values are means (± 1 S.E.) of 10 fully expanded, mature leaves per light environment.
Trait association and principal component analysis: The principal component analysis summarized the correlation structure of the nine morphological traits into three components, which explained 82.88 % of the variation (Table 2). Fenestrated area, effective leaf area, and leaf perimeter dominated the first component (39.14 %); these are traits associated to leaf size and shape. The second component (25.44 % of the variation) was dominated by lobulation ratio, stomatal density, and SLA (SLA was inversely related to the first two variables). The third component (18.30 %) showed high loadings for leaf width and petiole length.
Table 2 Principal component analysis summarizing the correlation structure of 9 leaf morphological characters in Monstera deliciosa. In bold-face variables dominating a given component.
| Principal component 1 | Principal component 2 | Principal component 3 | |
| Eigenvalue | 3.523097 | 2.28 | 1.64 |
| Percentage of variation | 39.14 | 25.44 | 18.30 |
| Cumulative percentage of variation | 39.14 | 64.58 | 82.88 |
| lnSD | 0.29 | -0.46 | -0.15 |
| Lnpetiole-lenght | 0.26 | 0.30 | 0.54 |
| Lnleaf-width | 0.31 | 0.20 | 0.54 |
| Lnleaf-lenght | 0.21 | 0.28 | -0.36 |
| Lnfenestrated-area | 0.48 | -0.18 | 0.0029 |
| Lneffective-leaf-area | 0.40 | 0.30 | -0.288 |
| Lnleaf-perimeter | 0.44 | -0.13 | 0.058 |
| Ln-SLA | -0.30 | 0.44 | 0.092 |
| lnlobulation-ratio | -0.18 | -0.48 | 0.40 |
The PCA used the ln-transformed values of the variables. SD = stomatal density, SLA = specific leaf area.
We ran a one-way MANOVA testing differences between sun and shade leaves across the scores of the first three principal components. We found a strong effect of habitat differences in the scores of the principal components (Hotelling-Lawley Trace3.16 = 4.74, p < 0.001), with significant differences for the first (F1.18 = 8.04, p < 0.01) and second components (F1.18 = 17.15, p < 0.0001, Fig. 2, Fig. 3). Differences among light environments were not significant for the third component (F1.18 = 0.54, p = 0.47).
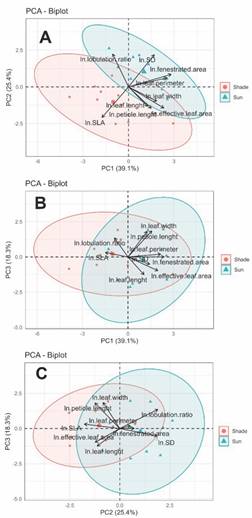
Fig. 2 Principal component analysis applied to nine ln-transformed morphological traits in Monstera deliciosa according to light environment. Ellipses show 95 % confidence intervals. (A) The first component was dominated by fenestrated area, effective leaf area and leaf perimeter, whereas the second component was dominated by stomatal density and lobulation ratio which maintained a negative correlation with SLA. (B) The third component was dominated by petiole length and leaf width. The first and second component separated sun and shade leaves. SD = stomatal density, SLA = specific leaf area.
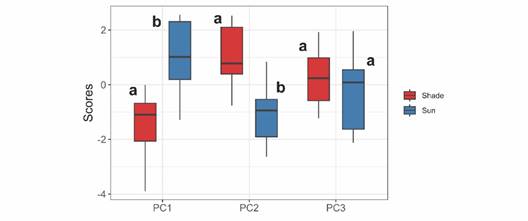
Fig. 3 Scores of three principal components based on the combined variation of nine Ln-transformed morphological traits in Monstera deliciosa across sun and shade light environments. Paired comparisons reflect the scores for sun and shade leaves within each component, which together explained 82.88% of the variation. Different letters indicate significant differences, while the same letter denotes a lack of significant differences.
Test of prediction a: mature sun and shade leaves will vary in fenestrated area and lobulation ratio, which will be higher in sun leaves.
Post hoc one-way ANOVAs were conducted for fenestrated area and lobulation ratio, using ln-transformed values to meet normality and homogeneity of variance assumptions. Fenestrated area showed higher values in sun leaves (F1.18 = 12.74, p < 0.001), whereas differences were not significant for the lobulation ratio (F1.18 = 0.7, p > 0.05).
Test of prediction b: sun leaves will have higher stomatal density and lower SLA than shade leaves.
Similarly, post hoc one-way ANOVAs were conducted for stomatal density and SLA, using ln-transformed values to meet assumptions of normality and homogeneity of variance. We found higher stomatal density in sun leaves (F1.18 = 60.86, p < 0.0001), and higher SLA values in shade leaves (F1.18 = 109.4, p < 0.0001).
Discussion
Monstera deliciosa exhibits distinct leaf phenotypes under sun and shade conditions. Sun leaves had a larger effective leaf area, more fenestrated area, a higher fenestration ratio, greater leaf perimeter, higher stomatal density, and lower SLA compared to shade leaves. The first principal component was primarily dominated by effective leaf area, leaf perimeter, and fenestrated area, which correlated with stomatal density and SLA. When examined separately, these traits (except SLA) were all higher in sun leaves, supporting our initial prediction of increased fenestration and stomatal density in sun leaves (and lower SLA in sun leaves). However, the fenestrated area comprised only a small proportion of the effective leaf area.
No significant differences in lobulation ratio were observed between sun and shade leaves, indicating a similar degree of dissection. Sun and shade leaves also had a similar total area and effective leaf area. This suggests that differences between sun and shade leaves extend beyond size and shape and are mostly determined by structural and functional traits, such as higher stomatal density and fenestrated area in sun leaves and higher SLA in shade leaves.
As leaf size increases, so does the area of fenestrations and the leaf perimeter, so that larger leaves have more fenestrations, and proportionally larger perimeter due to correlated growth. Also, it might seem contradictory that the fenestrated area and the leaf perimeter were decoupled from the lobulation ratio. We attribute this discrepancy to the fact that the lobulation ratio is correlated primarily with the amount of leaf area, whereas the fenestrated area and the leaf perimeter are also indicative of leaf shape. Therefore, while leaf size is an important morphological trait, it may not fully capture the subtle variation associated with the adjustment to light gradients mediated through changes in leaf shape (see Li et al., 2020) and structure (i.e., SLA, Kidner & Umbreen 2010). Our study analyzed only one leaf per plant, which limited our ability to assess whether the light intensity affecting that leaf influenced its morphology, structure, and size independently of the light conditions experienced by the rest of the crown, as affected by the plant’s resource allocation strategy (Francis & Gilman, 2019).
The fenestrated area, despite its small magnitude relative to total leaf area, increased in sun leaves, along with stomatal density. It is plausible that sun leaves are likely subject to higher hydraulic demands (López-Portillo et al., 2000; Muir, 2013). More dissected leaves (i.e., compound leaves) are more common in hot and dry environments at the top of the canopy (Givnish, 1979; Muir, 2013; Nicotra et al., 2010). As more fenestrations were associated to higher stomatal density, leaf thermal regulation is likely achieved through an increased fenestrated area as well as through stomatal regulation. Stomatic conductance data is necessary to test this idea as well as a more detailed analysis of the structure and size of stomata and its association with leaf thickness and vascular architecture (Kidner & Umbreen, 2010; Pérez-Bueno et al., 2022).
The fenestrated area made a low percentage of the effective leaf area, which indicates that changes in leaf shape are subtle under contrasting light environments, even though the fenestrated area for sun leaves was twice that of shade leaves. Thus, it is likely that M. deliciosa modulates its adaptation to different light regimes as the leaf develops through small changes in leaf shape. Since lobulation ratio is the proportion of leaf perimeter over the square of effective leaf area it is possible that the lobulation ratio did not capture small changes in leaf dissection, which were possibly more related to the fenestrated area and to the leaf perimeter. Longitudinal data are required to better control for environmental variation during leaf development. Although M. deliciosa can produce new leaves in the shade, it is also possible that the leaves currently in the shade would have initially developed under sun conditions. This scenario may indicate a significant capacity for post-expansion acclimatization to low light, which has been rarely documented in canopy plants (Avalos & Mulkey, 1999; Avalos & Mulkey, 2014). Post-expansion acclimation occurs more readily in sun leaves, driven primarily by changes in photochemistry rather than structural adjustments (Brooks et al., 1996). The significant differences in SLA between sun and shade leaves suggest long-term adaptation to their respective light environments, supporting the idea that each leaf type developed specifically within its native conditions. However, validating this hypothesis would require a long-term monitoring study to track leaf crown development, measuring how leaves acclimate as they progress through a range of light conditions during growth.
The morphological and structural differences of sun and shade leaves in M. deliciosa (i.e., increased fenestrated area and stomatal density in sun leaves and higher SLA in shade leaves) underscore the plant’s capacity to modify its leaf phenotype to contrasting light environments. These findings highlight the importance of subtle leaf shape modifications and indicate a potential for post-expansion acclimation, especially in sun leaves, to optimize performance under varying light conditions.
We hope that the methods described here will serve as a basis to expand the analysis of the function of fenestrations and the influence of leaf shape and size on leaf function in Araceae vines, including other Monstera species with different degrees of fenestration. Further research along these lines will help to finally answer some of the most recurring questions on the functional role of leaf heteroblasty (Kidner & Umbreen 2010), such as the impact of fenestration on the internal crown light environment of M. deliciosa, as well as how changes in leaf structure and function, expressed over time, facilitate habitat colonization.
Ethical statement: The authors declare that they all agree with this publication and made significant contributions; that there is no conflict of interest of any kind; and that we followed all pertinent ethical and legal procedures and requirements. All financial sources are fully and clearly stated in the acknowledgments section. A signed document has been filed in the journal archives.

