


 Inglés (pdf)
 Articulo en XML
 Referencias del artículo

 Traducción automática
 Enviar articulo por email
 Citado por SciELO
 Similares en
SciELO
 uBio

 Permalink

Zooplankton accomplishes an important role in the dynamics of coral reef ecosystems (McKinnon, Richardson, Burford, & Furnas, 2007). They represent the link between primary producers and multiple trophic levels (Alldredge & King, 2009), participate in biogeochemical cycles (Roman, Furnas, & Mullin, 1990), and on pelagic and benthic fauna recruitment (Hughes et al, 2000; Grorud-Colvert & Sponaugle, 2009). Composed of holoplanktic species that form swarms near reef structures (Hammer & Carleton, 1979); meroplanktic species (early stages of benthic or nektic fauna); and demersal species, which emerge from the benthos and migrate towards the surface during the night (Robichaux, Cohen, Reaka, & Allen, 1981). In the Caribbean basin, coral reef zooplankton is essential for reef ecosystem functioning (Yoshioka, Owen, & Pesante, 1985).
However, there is still a gap of information in some parts of the Caribbean region, especially in countries between Belize and Panama. Along the Caribbean coast of Costa Rica, the largest fringing reef is located in Cahuita National Park. Yet, there is a scarcity of surveys focusing on the pelagic realm. Silva-Benavides (1986) found the greatest biomass and abundance of phytoplankton during the rainiest month. As expected, these months report the highest input of terrestrial nutrients. In this park, Morales and Murillo (1996) surveyed the abundance and composition of zooplankton monthly in 1984. Peaks of total abundance also coincided with the rainiest months, leading to the assumption that the nutrient input has a strong effect on the zooplankton community of Cahuita through the increase of primary production. Copepods dominated the zooplankton abundance, while fish larvae and crustacean larvae were the principal groups of the meroplankton (Morales & Murillo, 1996). This study aimed at estimating the seston biomass, abundance and composition of the coral reef zooplankton, and marine invertebrate larvae, at Cahuita National Park after a 25 years gap of zooplankton research.
Material and methods
Study site:
Cahuita National Park is located on the Southern Caribbean coast of Costa Rica (9°45’ N - 82°48’ W). The fringing reef consists of a main crest (5 km) along Punta Cahuita, and two inner crests, one in the Eastern side (Puerto Vargas) and the other in the Western side (Playa Blanca) (Cortés & Risk, 1985). Small patch reefs and seagrass beds are common in the lagoon. The main current flows in a Northwest to Southeast direction, with eddy formation. In order to compare this research with Morales and Murillo’s work (1996), the same four stations (Sts. 1, 2, 3, 4) were selected. In addition, two stations at Playa Blanca were selected to look at the influence of two small rivers inflows: Perezoso (St. 5) and Suárez (St. 6) (Fig. 1). Features of the stations are summarized in table 1.
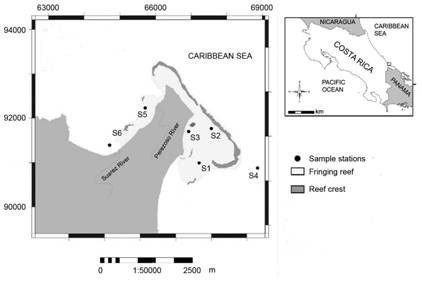
Fig. 1 Stations visited during September 2010-August 2011 at Cahuita National Park, Limón (modified from Fonseca, Salas, & Cortés, 2006).
Table 1 Morphological description of the stations sampled at Cahuita National Park, Limón, Costa Rica
| Station | Range of bottom depth (m) | Characteristics | Source |
|---|---|---|---|
| 1 | 4-6 | Back reef. Sandy bottom, coral rubble. Small colonies of Porites porites and Siderastrea siderea. | Morales & Murillo 1996; ACB, pers. Obs. |
| 2 | 2-3.5 | Back reef. Large colonies of Siderastrea siderea and Monstastrea complanata; benthic algae. | Morales & Murillo 1996; ACB, pers. Obs. |
| 3 | 1.5-2 | Back reef. Thalassia testudinum beds. | Morales & Murillo 1996 |
| 4 | 10-15 | Fore reef. Sandy and rocky bottom; benthic algae. | Morales & Murillo 1996 |
| 5 | 5-7.5 | Back reef. Thalassia testudinum and Syringodium filiforme beds; Manicina areolata colonies. | Nielsen-Múñoz & Cortés 2008; ACB, pers. Obs. |
| 6 | 4-6 | Back reef. Sandy bottom; Thalassia testudinum beds; large number of macroalgae (e.g. Sargassum). | ACB, pers. obs. |
Environmental features:
From September 2010 to August 2011, the salinity (Atago), surface sea temperature (SST) and Secchi depth were measured monthly at each station. Qualitative observations of cloud cover and surge were also obtained. The National Meteorological Institute provided data on precipitation and wind speed and direction (Table 2).
Table 2 Monthly mean of physical features during the zooplankton sampling in six stations at Cahuita National Park, Limón, Costa Rica; from September 2010 to August 2011
| Month | Sal (PSU) | Temp (°C) | Secchi Depth (m) | Prec. P.V. (mm) | Prec. Lim (mm) | Wind Speed Lim (km/h) |
|---|---|---|---|---|---|---|
| SET* | 34.2 | 29.3 | 3.6 | 145.2 | 90.1 | 7.4 |
| OCT* | 33.0 | 28.6 | 2.1 | 149.3 | 125.2 | 9.0 |
| NOV* | 35.5 | 28.9 | 3.5 | 372.2 | 592.8 | 8.4 |
| DEC* | 35.7 | 28.9 | 3.5 | 593.4 | 586.4 | 9.4 |
| JAN | 30.5 | 25.9 | 1.2 | 439.9 | 541.3 | 7.3 |
| FEB | 32.2 | 26.9 | 2.3 | 386.1 | 369.7 | 7.8 |
| MAR | 31.0 | 27.0 | 1.4 | 52.8 | 52.9 | 8.0 |
| APR | 31.5 | 25.9 | 1.4 | 184.7 | 222.1 | 8.1 |
| MAY | 32.0 | 27.5 | 3.6 | 360.7 | 406.6 | 8.0 |
| JUN | 29.7 | 29.3 | 5.6 | 208.2 | 190.2 | 8.0 |
| JUL | 31.3 | 29.4 | 2.8 | 212.6 | 140.1 | 7.4 |
| AUG | 32.7 | 29.1 | 3.5 | 35.6 | 62.0 | 7.1 |
*Months sampled in 2010. PSU: practical salinity units; Prec. P.V.: precipitation at Puerto Vargas; Prec. Lim: precipitation at Limón; Wind Speed Lim: wind speed at Limón.
Biomass and abundance:
During the year surveyed, two samples of zooplankton were collected monthly from each station, with the use of a Working Party (WP) net (0.47 m diameter opening and 200 µm mesh) for 5 min. Horizontal tows were conducted during daytime from a boat at 4 km/h. A calibrated flow meter (Model 2030R, General Oceanics, Incorporated) was attached to the net for later zooplankton abundance estimation. A buoy and a 2-pound weight were also attached to position the net to approximatly 1 m depth underwater. Stations were surveyed within 3 h during a given collection day.
Samples were fixed in a 4 % formalin/sea water solution. In the laboratory, no less than 72 h later, excessive detritus was removed from the samples using distilled water and 4 mm and 180 µm sieves. A Folsom splitter was used to obtain a subsample (1/4), from which seston dry weight was measured (Beers, 1981). Nakajima, Yoshida, Ross, & Toda (2010) suggested that zooplankton biomass is overestimated by the dry weight method in coastal ecosystems, due to high amount of phytoplankton and detritus. This is the reason why seston biomass was considered instead of zooplankton biomass for Cahuita. From another subsample, at least 400 organisms were counted and identified following Gasca & Suárez (1996), Smith and Johnson (1996), and Boltovskoy (1981).
A Canonical Correspondence Analysis was used to determine associations between the physical variables and the abundance of zooplankton groups, employing the MultiVariate Statistical Package (Kovach, 2004). Mean biomass (mg/m3) and mean total abundance (ind./m3) were transformed (log x + 1) to compare the stations and months sampled with an ANOVA in R version 3.1.0 (R Core Team, 2014).
A two-way ANOSIM evaluated the statistical differences in the abundance of different groups of zooplankton between months and stations, using PAST (Hammer, Haper, & Ryan, 2001). A one-way ANOSIM, with Gower distance was conducted to search for differences between Morales and Murillo (1996) and the present study. We selected the Gower distance because of the ordinal nature of some of the abundances reported by Morales and Murillo (1996). We used a MDS to show the differences. Finally, a paired t-test (or Wilcoxon for ordinal abundances) was performed to compare total zooplankton, holozooplankton, merozooplankton, and each zooplankton group’s abundance between both studies.
Results
Environmental conditions associations:
SST ranged from 25 to 30 ºC (mean= 28 ºC) and salinity from 27 to 37 PSU. The maximum depth of the Secchi disk was at St. 4, reaching 15 m in August 2011. Two peaks of precipitation were observed: one between November 2010 and February 2011, and the second one in May 2011. No clear association was found between the environmental variables, the months and stations sampled (Fig. 2A and Fig. B), except for a weak trend in the increment of precipitation in November 2010.
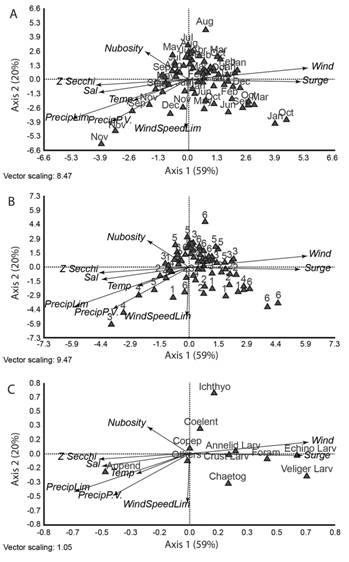
Fig. 2 Canonical correspondence analysis between environmental variables and (a) months, (b) stations and (c) general zooplankton taxa at Cahuita NP, Limón; from September 2010 to August 2011.
Between the zooplankton groups, the appendicularians showed an association with high values of precipitation, salinity and temperature. Some meroplankton forms like echinoderm or mollusk larvae were associated with wind and surge, the latter two environmental variables were strongly associated (Fig. 2C).
Seston biomass:
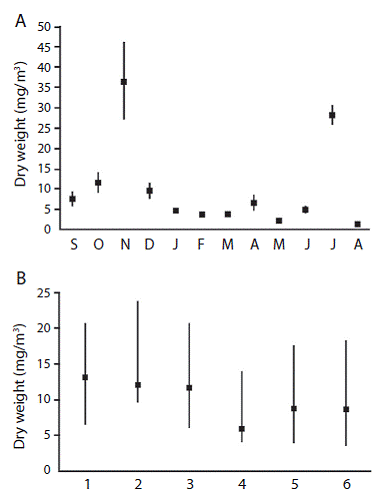
Seston biomass varied between months (Fig. 3A; ANOVA, P < 0.0001) from 0.49 mg/m3 (August 2011, St. 5) to 85.87 mg/m3 (October 2010, St. 2) with a mean of 10.05 ± 0.78 mg/m3. Highest seston values were observed for November 2010 and July 2011, whereas August 2011 showed the lowest record. Additionally, we found differences between stations (Fig. 3B; ANOVA, P < 0.05): St. 1, 2 and 3, as well St. 5 and 6 were very similar to each other, while St. 4 had the lowest biomass value.
Community abundance and composition:
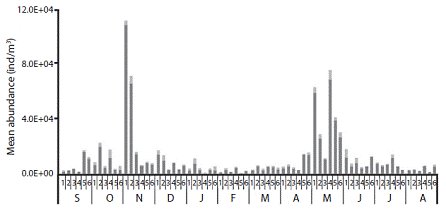
Zooplankton total abundance showed temporal and spatial variability, ranging from 1 145 ind./m3 (February 2011, St. 5) to 112 422 ind./m3 (November 2010, St.1), with a mean of 12 847 ± 510 ind./m3. Monthly differences were found (Fig. 4A; ANOVA, P < 0.0001), with two peaks: the first one in November 2010, that reached a mean abundance of 37 640 ± 44 293 ind./m3, and the second one in May 2011, reaching 42 402 ± 23 767 ind./m3. The lowest abundances were recorded in February 2011 (3 082 ± 1 746 ind./m3) and August 2011 (4 244 ± 1 955 ind./m3). Between stations the zooplankton abundance was also different (Fig. 4B; ANOVA, P < 0.05), with St. 1 and 2 possessing the highest abundances, and St. 3 the lowest.
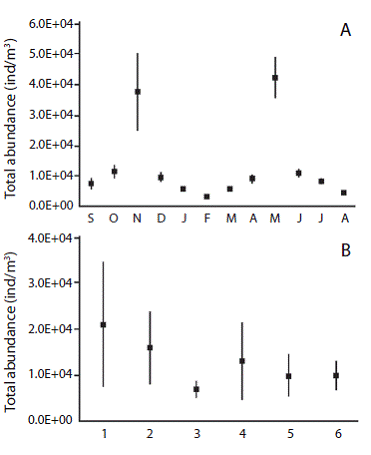
Fig. 4 Mean variation between months (a) and stations represent the se. (b) of zooplankton abundance at Cahuita NP, Limón; from September 2010 to August 2011. Error bars represent the se.
We found 38 taxa, which year-round showed significantly differences (ANOSIM, r2= 0.48; P < 0.0001). Zooplankton differed among stations (ANOSIM, r2= 0.44; P < 0.0001). Copepod abundance (8 431 ± 8 319 ind./m3) contributed 65 % of the total zooplankton abundance, with two peaks (November 2010 and May 2011) coinciding with the trends for total zooplankton abundance. Other notable groups include appendicularians and cladocerans which shows similar trends to these recorded in the zooplankton (Fig. 5). Among the meroplankton, mollusk and crustacean larvae (nauplii, mysis, zoea and phyllosoma) showed the highest abundances (Fig. 6). This led to a large difference between holoplankton and meroplankton abundance (Fig. 7).
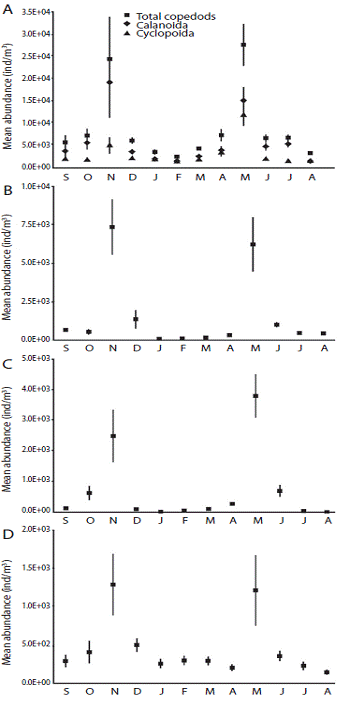
Fig. 5 Mean abundance of the dominant groups of holoplankton (a) copepods, (b) appendicularians, (c) cladocerans and (d) chaetognaths at Cahuita NP, Limón; from September 2010 to August 2011. Error bars represent the se.
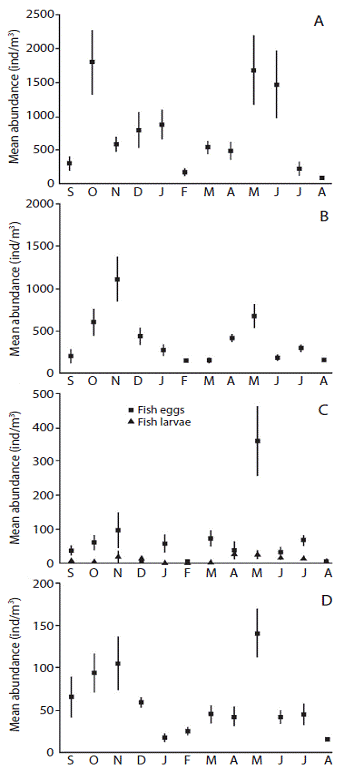
Fig. 6 Mean abundance of the dominant groups of meroplankton (a) mollusk veligers, (b) crustacean larvae, (c) ichthyoplankton and (d) polychaete larvae at Cahuita NP, Limón; from September 2010 to August 2011. Error bars represent the se.
Zooplankton community 25 years later:
Zooplankton abundances recorded in January and November were different than those reported by Morales and Murillo (1996) (ANOSIM, r2= 0.67, P < 0.001). The mean abundance (645 ± 84 vs 13 184 ± 4 104 ind./m3) was 20 times higher in the present study (Fig. 8), and the MDS evidently showed the difference (Fig. 9). Such differences resulted from the disparity between copepod and appendicularian abundances. These groups were respectively 63 and 170 times more abundant overall, and in November, 170 and 7 340 times, in the present study. The rest of the zooplankton groups also showed differences between studies, except for foraminifera, amphipods and icthyoplankton.
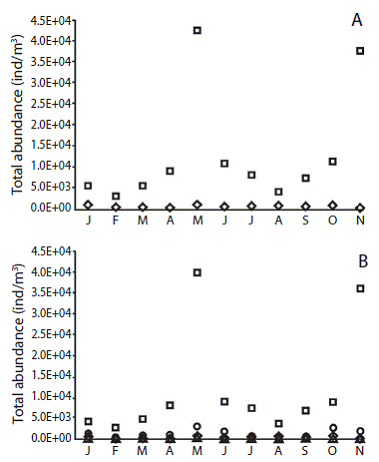
Fig. 8 (a) Total abundance of total zooplankton (squares: present study; diamonds: Morales & Murillo (1996)); (b) total abundance of holozooplankton (squares: present study; diamonds: Morales & Murillo (1996)) and merozooplankton (circles: present study; triangles: Morales & Murillo (1996)) of the months shared between Morales & Murillo (1996) and the present study at Cahuita NP, Limón.
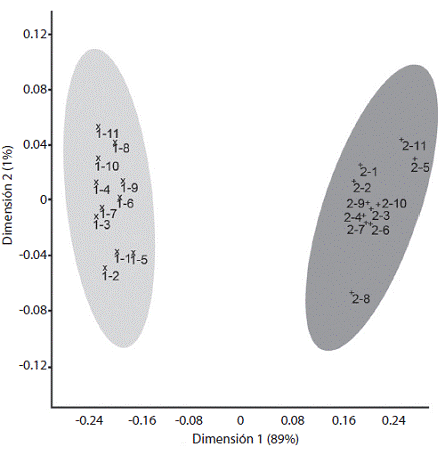
Fig. 9 MDS using Gower’s distance among general zooplankton taxa and the months and the stations shared between Morales & Murillo (1996) and the present study. Cahuita NP, Limón. Morales & Murillo (1996) data set represented by a number “1” in light gray and the present study represented by a number “2” in dark gray. Numbers after hyphen represents the month shared: from January (1) to November (11).
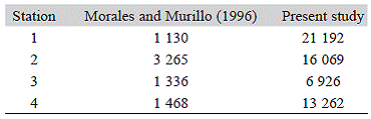
Shared stations (St. 1-4) also showed differences, being 29 times more abundant than those recorded by Morales and Murillo (1996) (ANOSIM, r2= 0.89; P < 0.05; Table 3). Higher abundance overall was found in St. 1 (21 192 ind./m3) and 2 (16 069 ind./m3). By contrast, in 1984, St. 2 and 4 were more abundant.
Table 3 Total abundance of zooplankton (ind./m3) from the shared stations between Morales and Murillo (1996) and the present study (September 2010-August 2011) at Cahuita NP, Limón
Discussion
Precipitation was associated with temperature, salinity and Secchi depth, but not with a particular station or month sampled. We expected that salinity would decrease in St. 5 and St. 6, both at river mouths. However, apparently their runoff does not contribute much to a decrease in either salinity or temperature.
Salinity and Secchi depth values were similar to those reported before (Silva-Benavides, 1986). The highest transparency and salinity recorded in St. 4 (outer crest) indicated the effect of a more oceanic condition. On the other hand, the sediment resuspension near the shoreline produces an input of nutrients to the water column, resulting in more food for planktic primary producers, but more turbidity for benthic primary producers.
We present the first values of seston biomass for Cahuita’s reef. Few seston biomass records for the Grand Caribbean are primarily available from Mexico. The seston values recorded in Cahuita (0.49-85.87 mg/m3) are lower than those recorded in Mahahual (14.79143.26 mg/m3) by Castellanos and Suárez (1997). On the North-side of Quintana Roo, a higher value (75 mg/m3) was found in a coastal lagoon system compared to the reef (36 mg/m3), but the latter was higher than in the ocean waters (34 mg/m3). This difference was attributed to higher nutrient resuspension rates (Álvarez-Cardena, Ordóñez-López, ValdésLozano, Almaral-Mendívil, & Uicab-Sabido, 2007). A relationship between higher concentrations of nitrates, chlorophyll a and zooplankton biomass, has been found in other Caribbean reefs like Bocas del Toro and Laguna Chiriquí in Panama (D’Croz, del Rosario, & Góndola, 2005) and Puerto Rico (Yoshioka et al., 1985).
The mean average zooplankton abundance recorded in this study (12 847 ± 510 ind./m3) exceeded the obtained values of other surveys in the Caribbean. For instance, those in Quintana Roo, México (8 808 ind./m3) (ÁlvarezCardena et al., 2007), Mahahual, México (64 ind./m3) (Castellanos & Suárez, 1997), and Jamaica (1317-3940 ind./m3) (Webber, Roff, Chisholm, & Clarke, 1996). Calanoid copepods dominated the Cahuita zooplankton community, as they do in the majority of the marine ecosystems (Hulsemann, 1996). Calanoids were more abundant in November 2010 (St. 1 and St. 2), while cyclopoids were more abundant in May 2011 (St. 1 and St. 4). For instance, in Jamaica, Ohlhorst (1985) demonstrated that the spatiotemporal variability of zooplankton is mainly the product of Oithona colcarva swarming.
Other groups like appendicularians and cladocerans contributed strongly to the abundance of the zooplankton community. Because of high growth rates, the appendicularian Oikopleura longicauda can surpass copepod production (Hopcroft & Roff, 1998). Also, the efficient grazing characteristics of the cladoceran Penilia avirostris enable it to achieve abundances of up to 2 500 ind./m3 (Rose, Roff, & Hopcroft, 2004).
Mollusk larvae dominated the meroplankton, with values higher than those reported from Mexico (Oliva-Rivera & de Jesús-Navarrete, 2000), where abundance peaks were associated with the rainy season and higher sea temperature. Morales and Murillo (1996) found the same dominance, but in the present study, we found no relationship between larval abundance and precipitation or temperature.
In addition to biomass, sediment resuspension has been correlated with high abundances of zooplankters in the Nichupte lagoon system (Mexico) (Álvarez-Cardena et al., 2007) and in the Great Barrier Reef (McKinnon et al., 2007). We found the highest abundances in Cahuita, near the shoreline of Puerto Vargas (St. 1 and 2), where previously Roder, Cortés, Jiménez and Lara (2009) reported high values of total suspended matter.
The higher total abundance in the present study, relative to the one documented by Morales and Murillo (1996), is caused by the holoplanktic groups. Copepod abundance was 32 times higher in the present study than in 1984. This is an underestimate of copepod abundance, as very abundant swarms of Oithona and Oncea are usually predominant in ocean waters, but are not retained by > 200 µm nets (Gallienne & Robins, 2001). Noticeably, Morales and Murillo (1996) used a 280 µm mesh size net, discriminating smaller components of the zooplankton that could explain such large differences. Previously, we reported new records of copepods found in the study (Morales-Ramírez, Suárez-Morales, CorralesUgalde, & Esquivel-Garrote, 2014), plus the description of two new species of monstrilloid copepods: Monstrillopsis cahuitae SuárezMorales, Carrillo and Morales-Ramírez, 2013 and Cymbasoma alvaroi Suárez-Morales & Carrillo, 2013 (Suárez-Morales, Carrillo, & Morales-Ramírez, 2013). Following the same trend, appendicularian and mollusk larvae (meroplankton) abundance was also too low in the past study relative to our current measures.
What are the causes of this divergence in the total and particular abundance of zooplankters between both studies? As mentioned before, the resuspended sediments have been correlated with peaks of biomass and abundance (Álvarez-Cardena et al., 2007). In Cahuita, Roder et al. (2009) found four times more total suspended material in 2004 and 2005 than Cortés and Risk (1985) did in the 1980’s. In addition, we found the highest concentrations in Puerto Vargas site, which coincides with peaks of abundance and biomass.
Cortés and Risk (1985) demonstrated that terrestrial runoff from the La Estrella and Banano Rivers adversely affects the health of the reef at Cahuita. In recent years, several land-use changes could be the responsible for a larger discharge of nutrients and silt in those rivers (Mora-Cordero & Chavarría, 2009).
Moreover, the 1982-1983 ENSO could have triggered certain anomalies in the Caribbean Sea and the Equatorial Atlantic Ocean (González et al., 2000). On the Pacific coast of Costa Rica, Quesada-Alpízar and MoralesRamírez (2006) found a lower zooplankton abundance and biomass during the 1997 ENSO. González et al. (2000) reported an increase in the wind speed, precipitation and surge in the Caribbean coast of Mexico. Hence, these effects might be expected to produce an increase in the zooplankton abundance, rather than the decrease seen in Cahuita. This leads us to think that the 1982-1983 ENSO cannot explain the low abundances reported by Morales and Murillo (1996).
Most of the coral reefs are composed of sessile benthic organisms with a planktic larval phase important for dispersion, spatial distribution stabilization and gene flow (Poulin, Boletzky, & Féral, 2001). At Cahuita, the meroplankton does not exceed the abundance and diversity of the holoplankton. However, among the essential components in a coral reef, a diverse range of larval forms were found. We also found a high diversity in polychaete larvae and the occurrence of lophophorate larvae. Cahuita seems to have a high availability of larvae, and hence, of possible recruits for the reef.
The coral reef in Cahuita is only an example of the degradation that coral reefs have suffered over the past 30 years (Cortés et al., 2010). Mostly siltation has affected the amount of light available for photosynthesis and also had smothered the living corals, leading to a low growth and low development. However, the high abundance of zooplankton found in this study indicates that nutrient input and zooplankton recruitment are important sources that enable the permanency and survival of corals and reef fauna. Studies of feeding dynamics and elaboration of trophic models are necessary to elucidate the role that zooplankton can have in coral reef resilience, not only in Cahuita National Park but for the entire Caribbean coast of Central America.

